Altitonans_Fulmen The thoughts shared in this journal are my own—a snapshot of personal understanding at the exact moment of writing. It is not intended as a reference of absolute fact, but rather as an exercise in ἐπίνοια (epinoia): an exploration of thought, intuition, and creative insight.
Epinoia(ἐπίνοια) is a Greek term meaning thought, intention, purpose, or conception, stemming from "mind" (nous) and "upon" (epi), representing the mind's reflective or creative process, used in philosophy (Aristotle, Gnosticism) and theology to discuss understanding and divine names, appearing once in the New Testament for the "intent of your heart" (Acts 8:22). It signifies the mind's operation to form ideas or designs, contrasting with raw data or innate perception, and in Gnosticism, it's an emanation of divine wisdom (Sophia).
"Φsis" is a stylized spelling of the Ancient Greek word φύσις (physis), which translates directly to "nature" or the intrinsic essence of a living thing.
Exploring the deep intersection of science, intuition, and creative insight often leads to breakthroughs that challenge our understanding of what is possible. When we approach high-performance cultivation not just as a hobby, but as an exercise in pushing a biological system to its absolute genetic ceiling, the results can transform from simple data points into profound proof of concept. Achieving a highly optimized environment requires a shift in mindset away from empty promises and directly toward verifiable proof, building true confidence through a detailed archive of past lessons and strategic adjustments.
This philosophy turns a standard space into a precise mass and energy balance equation, where every variable is managed to eliminate biological bottlenecks entirely. In a recent project four individual plants produced 344 grams, 280 grams, 445 grams, and 255 grams respectively, resulting in a total harvest of 1,324 grams, or 47.2 ounces, of dry product. Operating with a 600-watt light source inside a four-by-four footprint, this brings the final efficiency to an exceptional 2.21 grams per watt.
To put this in perspective, the standard traditional indoor benchmark has long been established at 1.0 grams per watt, while expert commercial operations target 1.5 grams per watt, and elite commercial systems push the envelope between 1.8 and 2.0 grams per watt. Reaching 2.21 grams per watt places the outcome squarely within the top 0.1 percent of global benchmarks, acting as a true statistical outlier that demonstrates what happens when flawless environmental parameters meet a cultivar pushed to its maximum potential. Reaching this level of mastery demands that we move past the common trap of the mirror fallacy, where the ego mistakes its own limited perspective for universal truth and views different ideas as personal threats. True progress requires curiosity and dismantling the illusion that our immediate viewpoint is the objective standard, shifting the focus instead toward how a system actually operates under the absolute laws of physics. In a high-performance setup, maximizing output is never about adding random additives or forcing growth, but rather about systematically removing the limitations that hold the organism back. By maintaining a perfect vapor pressure deficit, ideal root-zone oxygenation, and precise structural canopy training every single minute of the cycle, the plant is freed to express 100 percent of its DNA potential without any lingering genetic latency.
Managing a dense canopy inside a tight footprint presents the ultimate challenge of mitigating stagnant air and preventing moisture issues. Overcoming this bottleneck relies on a sophisticated synganic approach, which seamlessly marries the precise control of synthetic mineral inputs with the natural resilience of active organic living soil. This method transforms the room into a closed-loop system where the internal microclimate is entirely isolated from external weather fluctuations and pests. Rather than openly exhausting the atmosphere, the air is continuously recirculated, enriched, and scrubbed using 264-nanometer ultraviolet light.
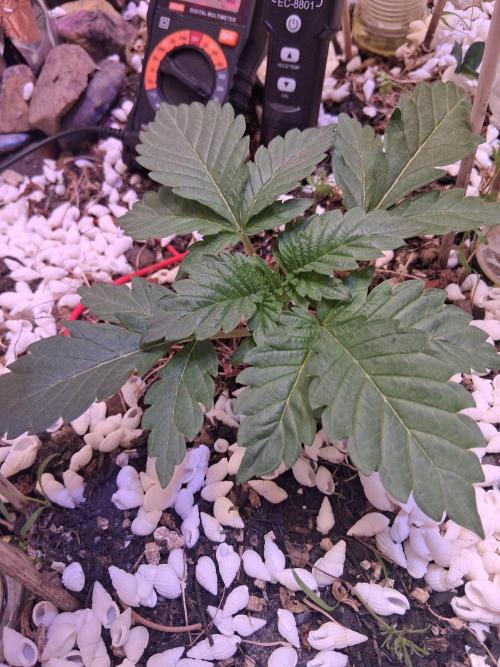
The foundation of this thriving ecosystem is a comprehensive substrate composition designed to provide perfect aeration, structural integrity, and biological buffering. The primary media base integrates expanded clay aggregates, coir chunks, premium coco coir, sphagnum peat moss, horticultural perlite, vermiculite, pumice, and volcanic basalt rock. To continuously condition the soil and fine-tune mineral availability, the mixture is amended with agricultural gypsum, wollastonite, dolomitic limestone, basalt rock dust, micronutrient-rich volcanic ash, greensand, crushed seashells, biochar, and shungite. This mineral architecture creates an incredibly stable environment where active soil biology naturally prevents salt toxicity and ensures steady, reliable nutrition throughout the entire life cycle.
Living organisms within the substrate play a vital role in maintaining this delicate biological balance and breaking down organic material. Red wigglers continuously process organic matter into easily accessible plant nutrients while aerating the media; specialized predatory mites offer excellent biological control against common soil pests, and pillbugs excel at breaking down tough, woody elements. These biological components are further supported by a rich layer of organic amendments including high-phosphorus steamed bone meal, high-nitrogen dehydrated blood meal, fish bone meal, cold-processed kelp meal, dehydrated moringa powder, spirulina powder, and marine crustacean biomass rich in chitin. Combined with biological inoculants like mycorrhizal fungi, premium worm castings, and concentrated humic and fulvic acids, the entire system operates as a flawless biological transducer of light and energy.
Ultimately, shifting our perspective to view a grow space as a complete mass and energy balance equation changes the entire nature of agriculture. Success ceases to be a matter of luck or anecdotal habits and instead becomes the predictable result of meticulous design, patience, and the strategic elimination of failure. When science, biology, and engineering converge so harmoniously, we gain a deeper appreciation for the intricate natural systems that sustain life and growth. By sharing these detailed insights and refining our techniques, we can continue to unlock the absolute maximum potential hidden within the living world around us.
Comprehensive Substrate Composition:
1. Substrate Base & Aeration Media
Expanded Clay Aggregates (Hydroton Pebbles)
Coir Chunks & Horticultural Coco Coir
Sphagnum Peat Moss
Horticultural Perlite
Horticultural Vermiculite
Horticultural Pumice
Volcanic Basalt Rock
2. Mineral Amendments & Soil Conditioners
Agricultural Gypsum (Calcium Sulfate)
Wollastonite (Calcium Silicate)
Dolomitic Limestone (Calcium Magnesium Carbonate)
Basalt Rock Dust (Trace Mineralizer)
Azomite (Micronutrient-Rich Volcanic Ash)
Glauconite (Greensand)
Crushed Seashells (Calcium Carbonate Source)
Pyrolyzed Carbon Feedstocks (Biochar & Horticultural Charcoal)
Elite Shungite (Carbonaceous Mineraloid)
3. Organic Nutrient Amendments
Steamed Bone Meal (High Phosphorus)
Dehydrated Blood Meal (High Nitrogen)
Fish Bone Meal (Phosphorus & Trace Calcium)
Cold-Processed Kelp Meal (Ascophyllum nodosum)
Dehydrated Moringa Oleifera Powder (Botanical Nutrient)
Spirulina Powder (Arthrospira platensis / Cyanobacteria Nutrient)
Marine Crustacean Biomass (Shrimp & Crab Chitin)
4. Biological Inoculants & Organic Acids
Mycorrhizal Fungi Inoculant (Endomycorrhizae / Ectomycorrhizae)
Vermicompost (Premium Worm Castings)
Humic & Fulvic Acids (Concentrated Humates)
Human Body
65% Oxygen (in all liquids and tissues, bones, and proteins)
18% Carbon (everywhere)
10% Hydrogen (in all liquids and tissues, bones, proteins
3% Nitrogen (in all liquids and tissues, proteins
1,5% Calcium (lungs, kidney, liver, thyroid, brain, muscles, heart, bones)
1% Phosphorus (urine, bones, DNA)
0,35% Potassium (enzymes)
0,25% Sulphur (proteins)
0,15% Sodium (in all liquids and tissues) (in terms of salt)
0,05% Magnesium (lungs, kidney, liver, thyroid, brain, muscles, heart)
Plant
Mother-nutrients: Carbon 47%, Oxygen 43%, Hydrogen 4%.
Macro-nutrients: Nitrogen 3%, Phosphorus1%, Potassium1%, Calcium1%, Magnesium0.5%, Sulfur0.5%.
Micro-nutrients: All the rest combined 1%
More energy, more blueprint.
Although CO2 is a naturally occurring gas that both humans and plants use, it is invisible and odorless and can be fatal at high-levels. If you’re supplementing carbon dioxide in your grow room, ensure there are no leaks in any CO2 devices and always use a CO2 monitor and alarm.
0.02% Life unsustainable
0.03% Life OK
0.04% Current ambient atmospheric co2
0.04%-0.1% =400-1000ppm standard indoor co2.
0.1%-0.2% = 1000- 2000 ppm (prolonged exposure: drowsiness).
0.2%-0.4% = 2000-4000ppm (Headaches, fatigue, stagnation, stuffiness, poor concentration, loss of focus, increased heart rate, nausea).
1% is toxic
5% is quick death.
"Dabo vobis quod oculus non vidit, nec auris audivit, nec manus tetigit, quod in cor hominis non ascendit."
5 likes
comments
Share
1
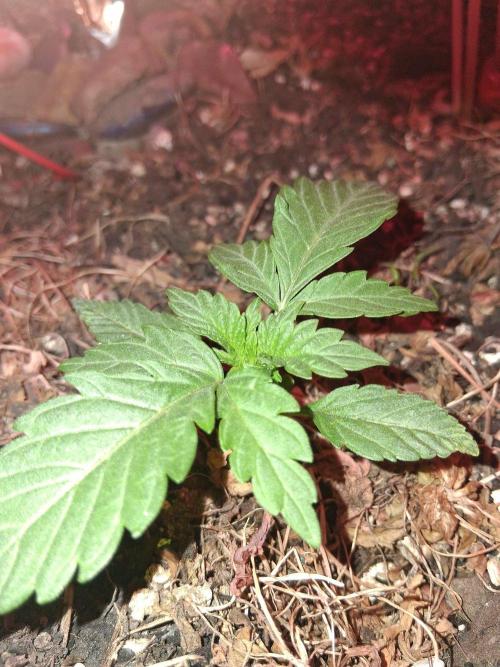
Week 1. Vegetation
12d ago
1/30
10.16 cm
Height
18 hrs
Light Schedule
24 °C
Day Air Temp
137.16 cm
Lamp Distance
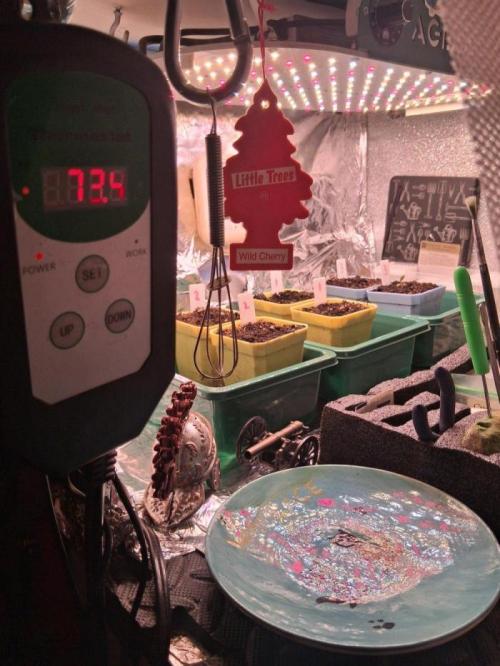
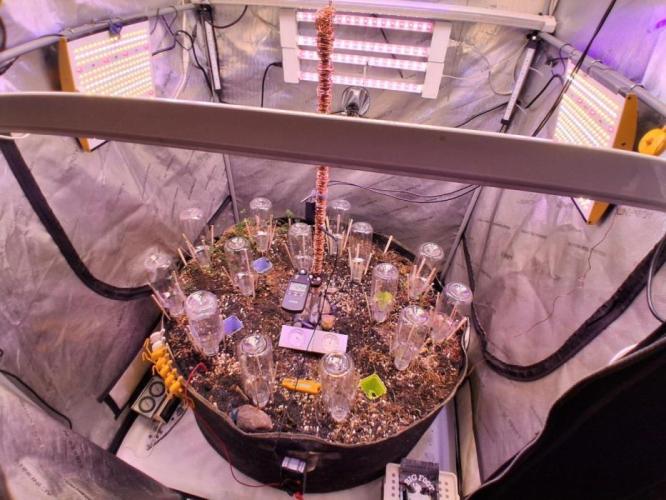
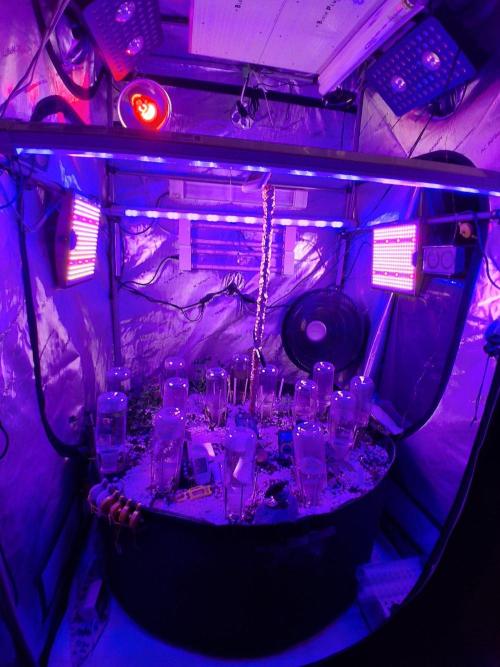
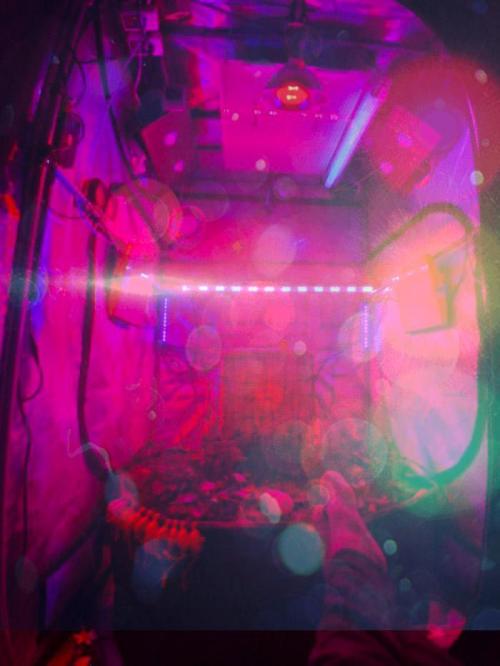
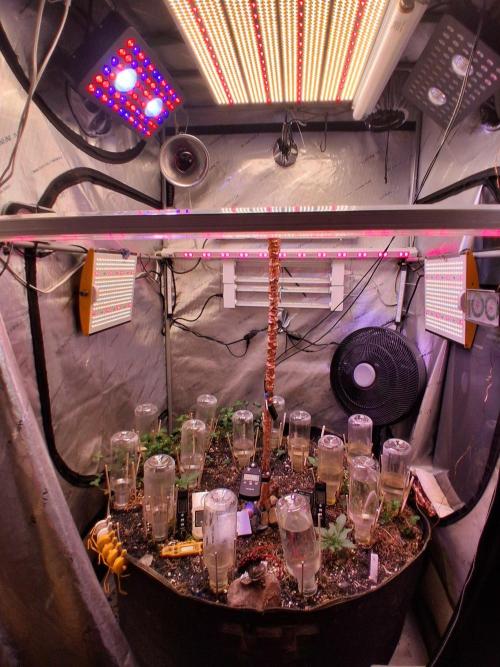
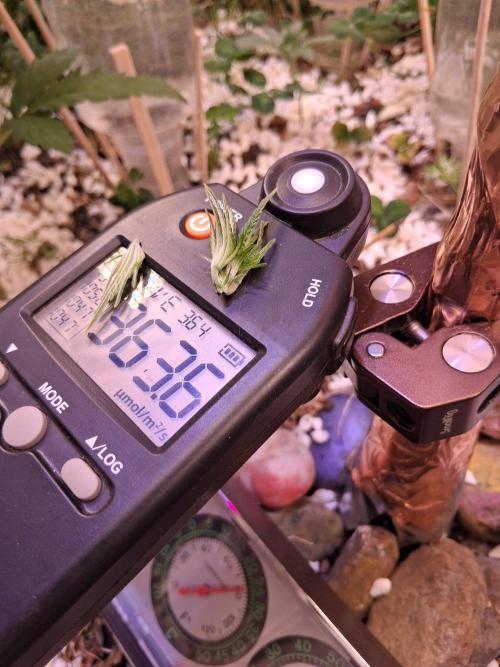
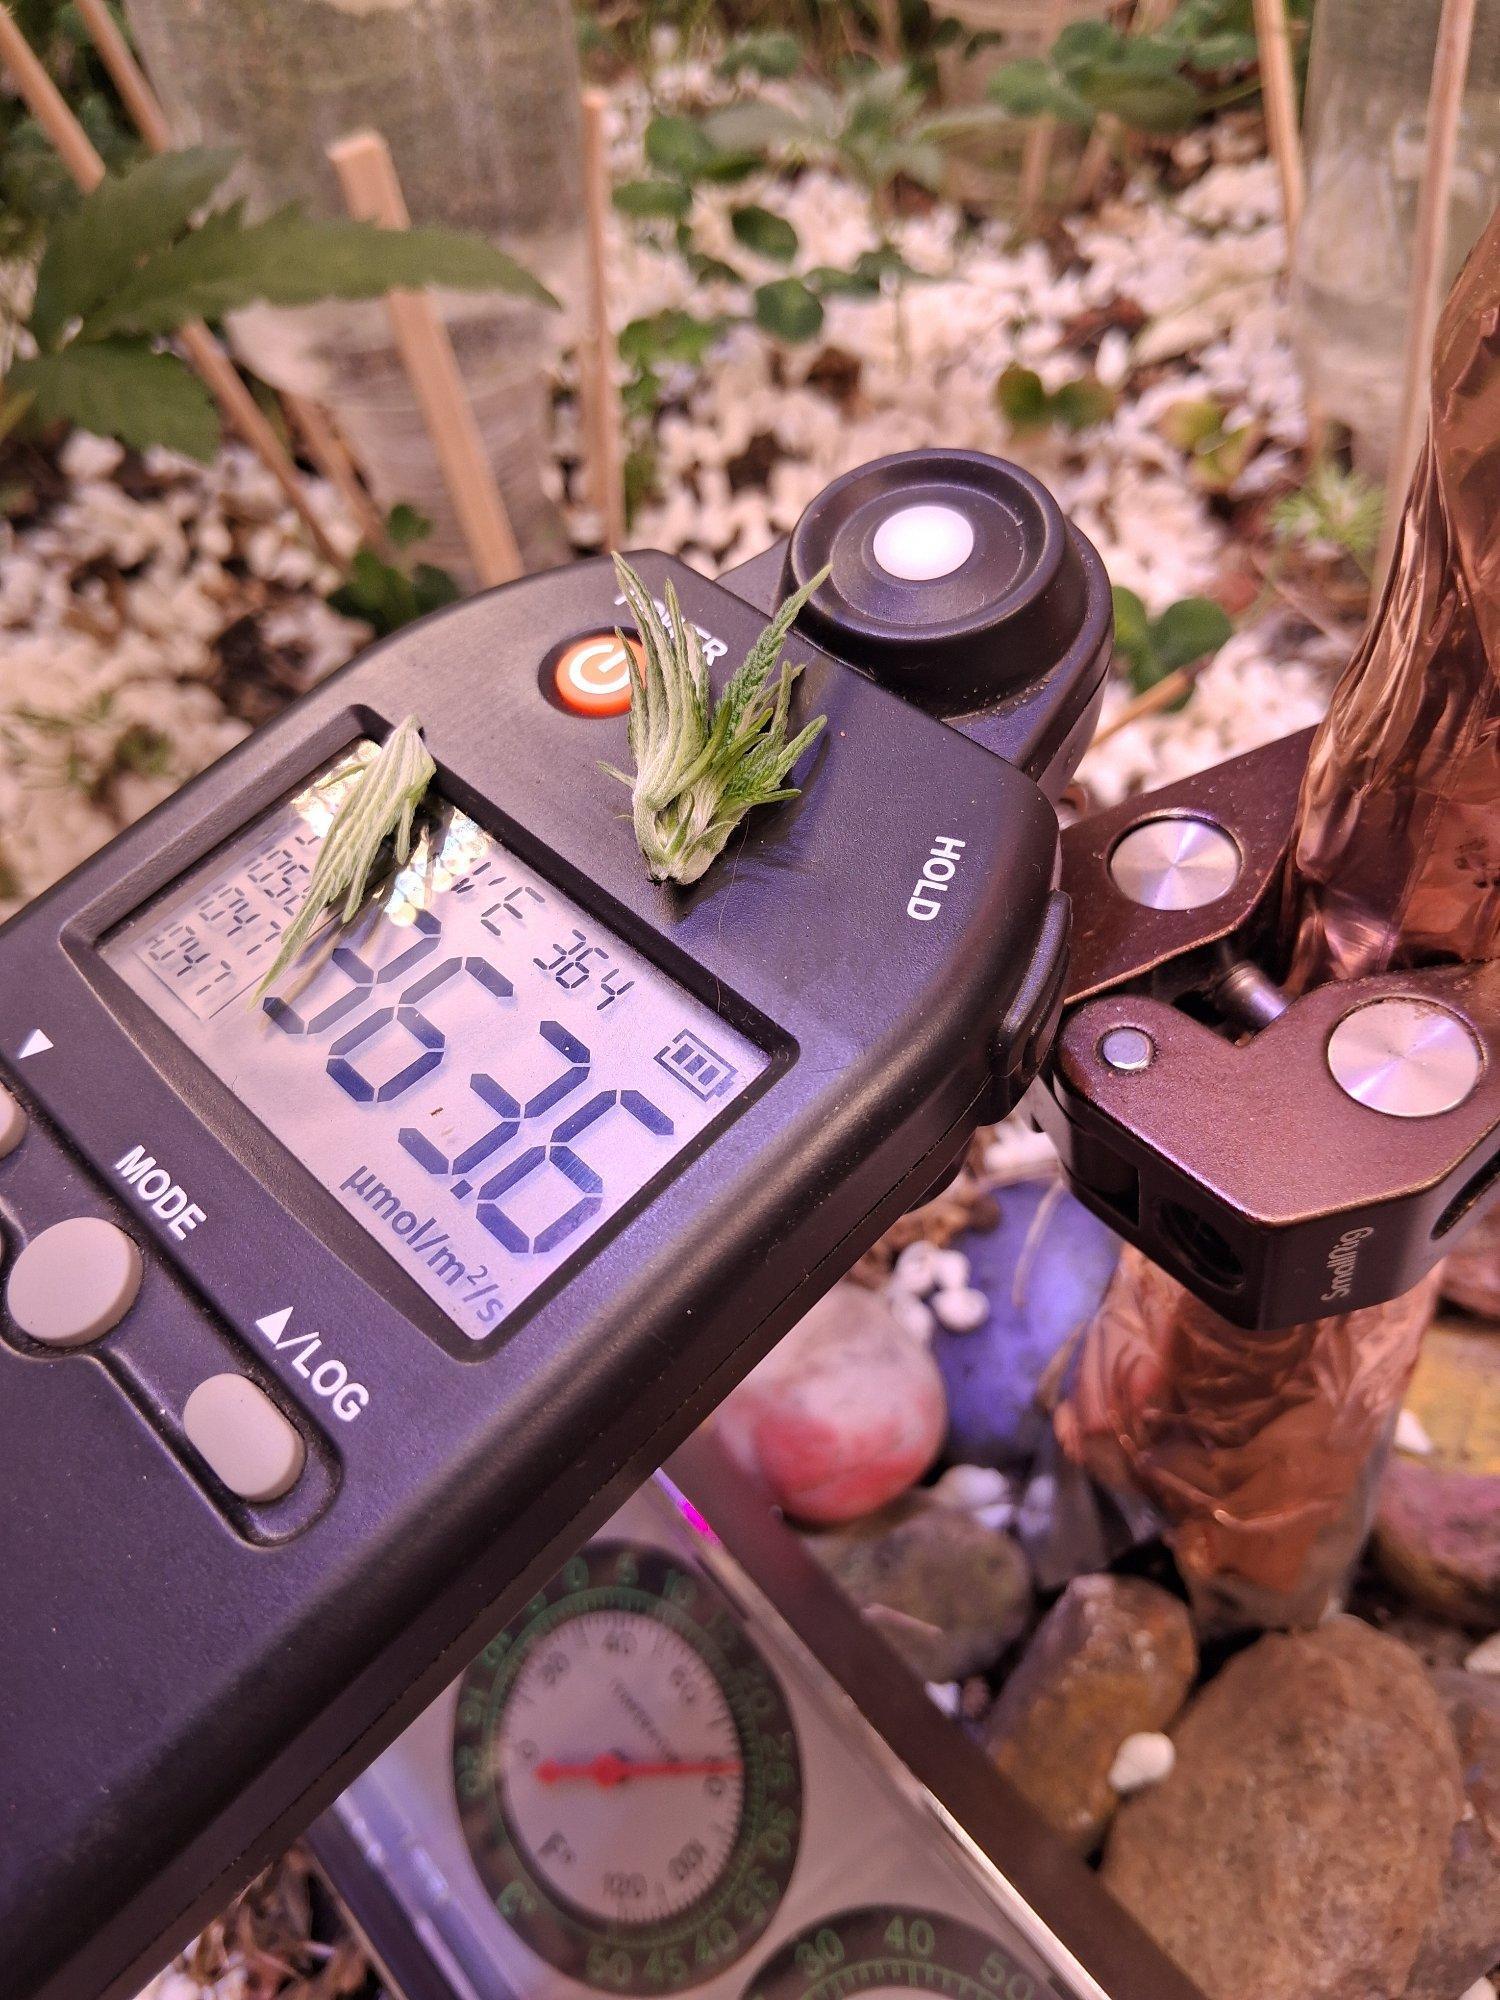
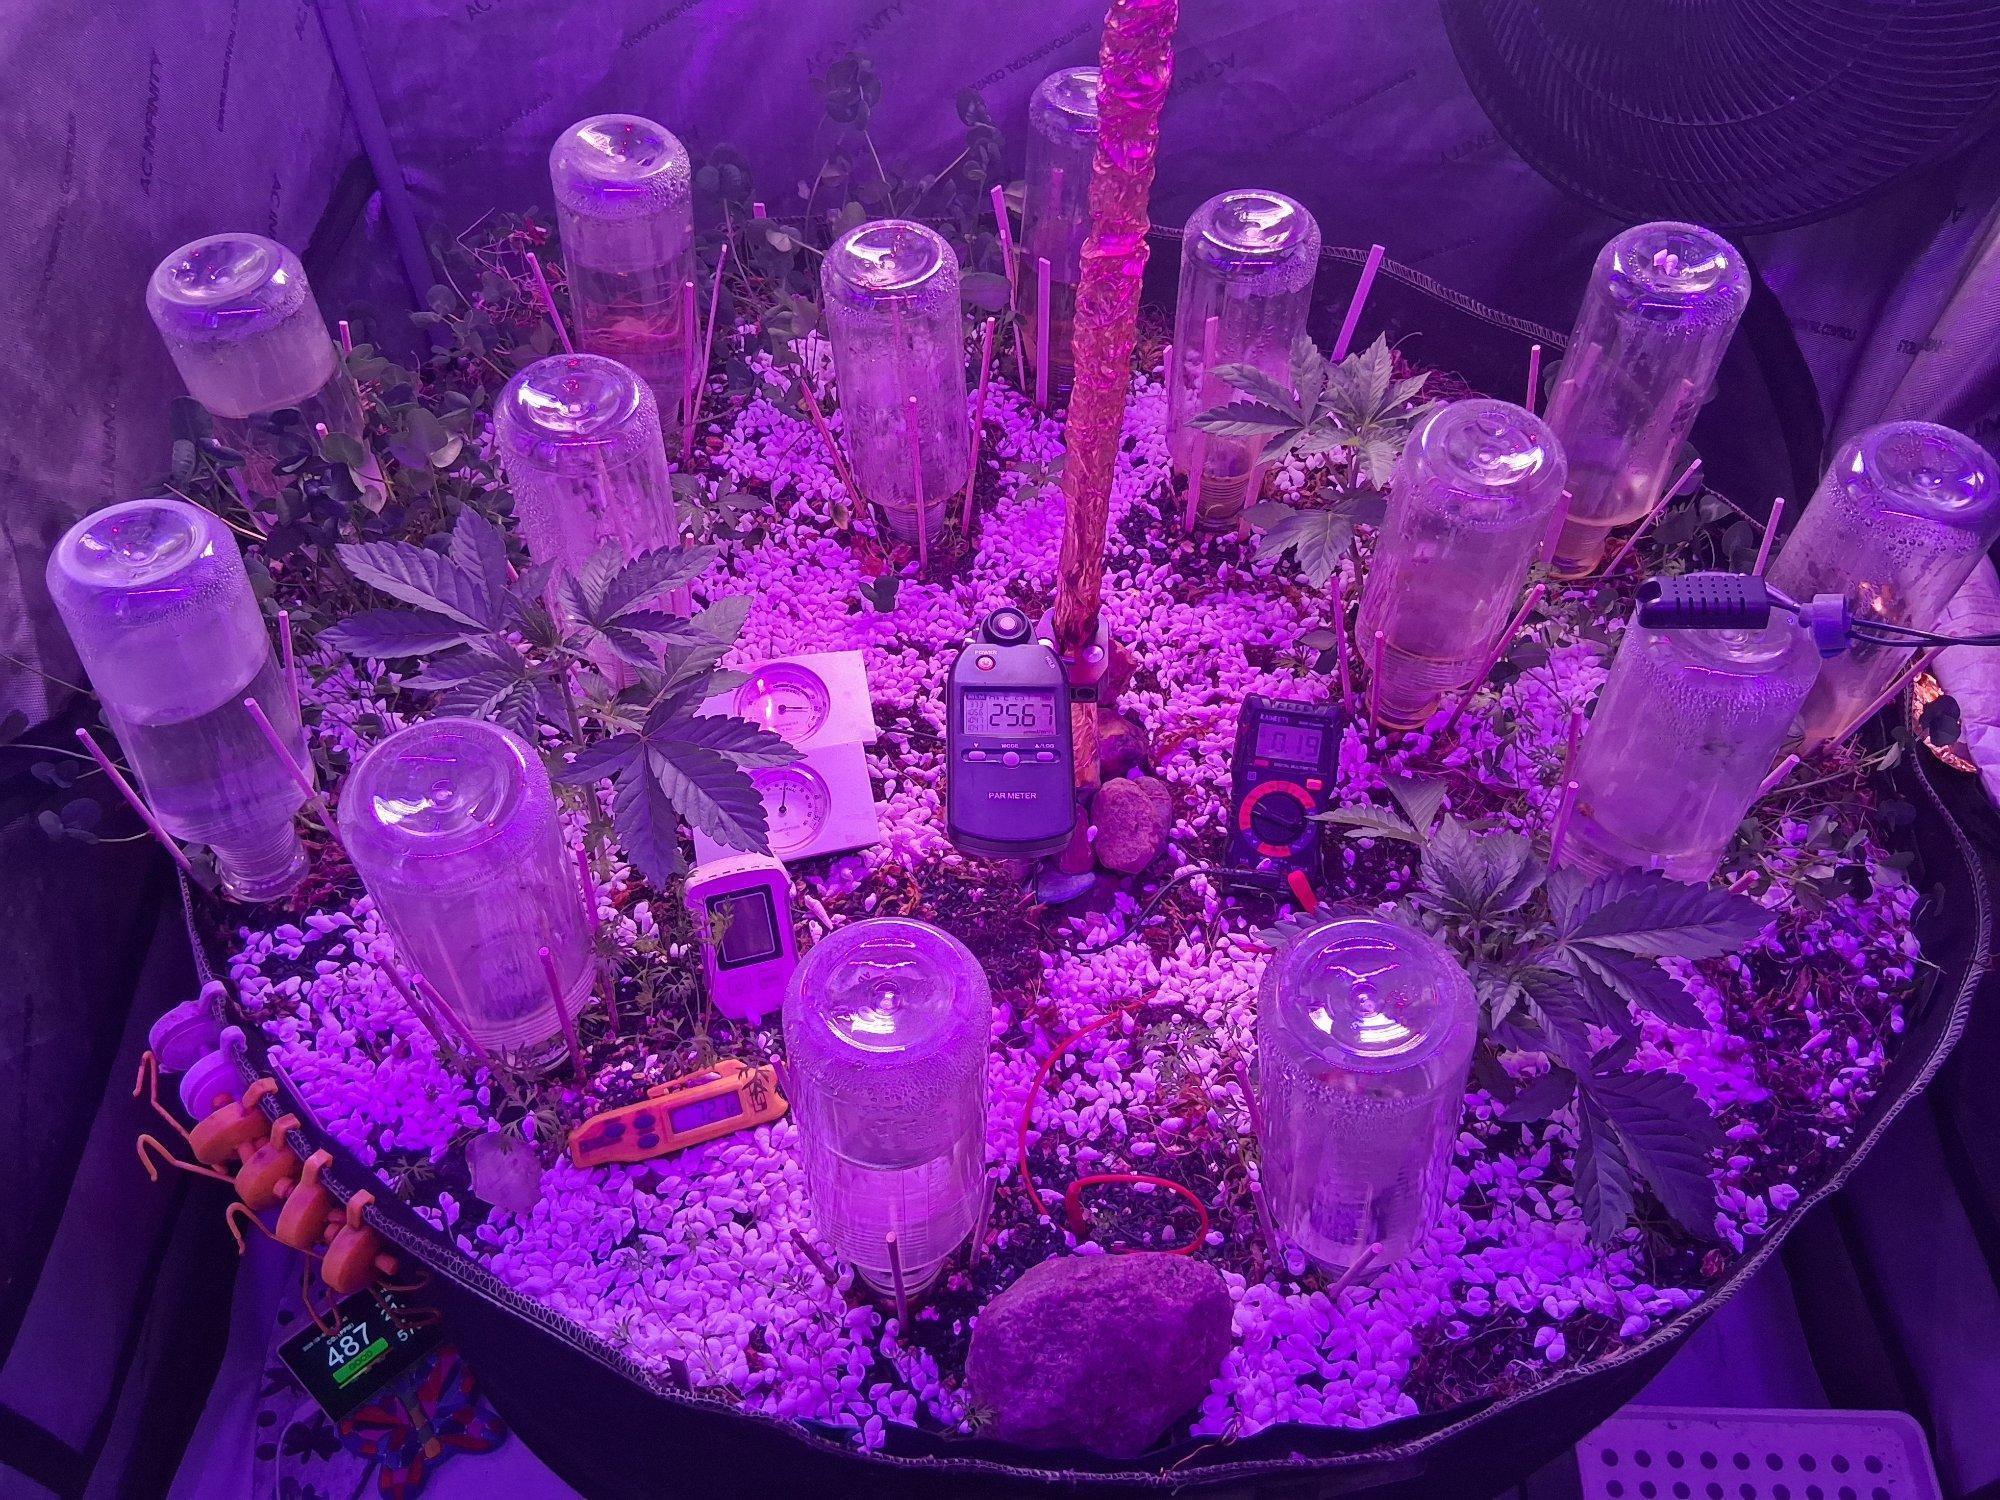
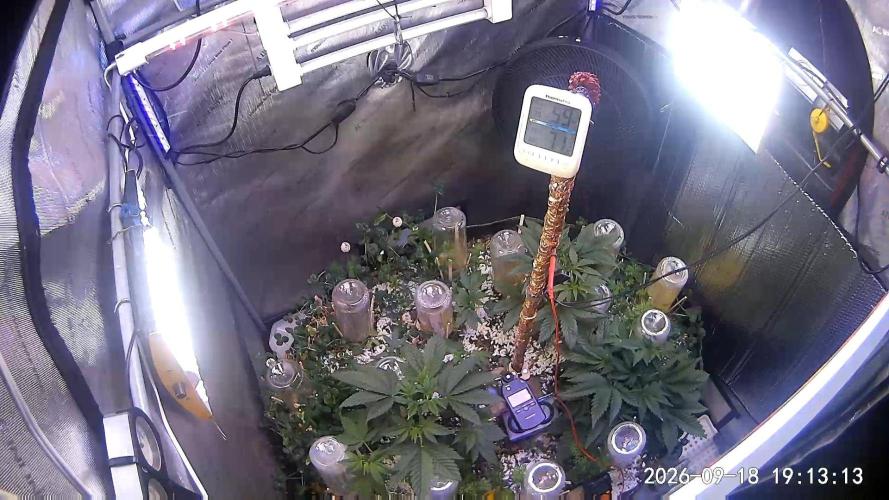
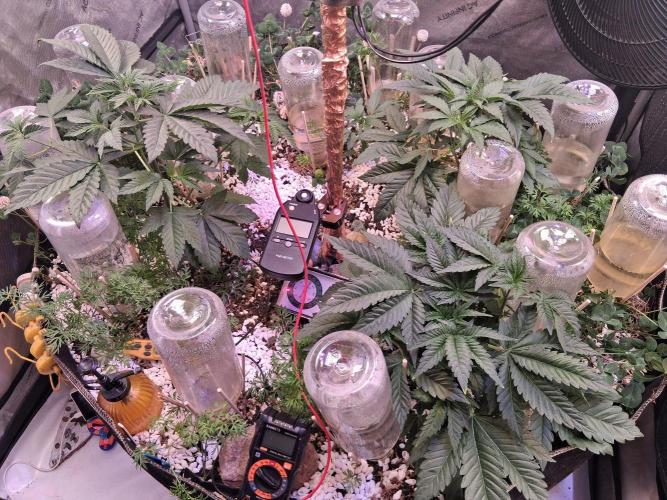
Altitonans_Fulmen Lights are 58 inches from the main source to the top of the pot and the soil surface. If you added up all the lights in the tent, it would be 1100w-1200w total across 14 lights. Using them all at once is far too much for a plant and incredibly difficult to deal with environmentally. The lights are fixed in position; side lights have dimmers, allowing for pinpoint precision of PPF. Fixed at 58 inches, cannot move them closer to increase intensity. Instead, achieve optimal PPF by distributing smaller wattages across a massive, multi-fixture matrix. Triggering specific plant defenses without melting the canopy.
What's the point/blah blah wattage?
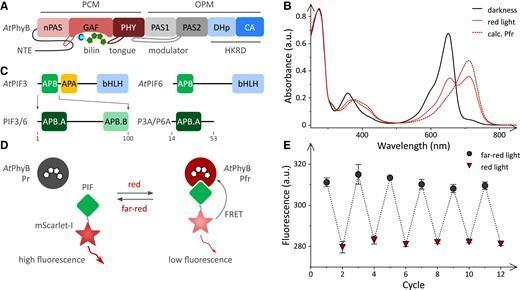
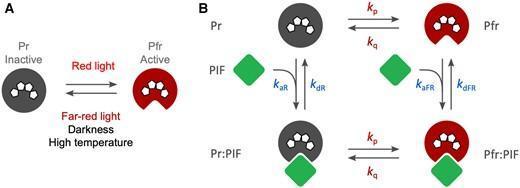
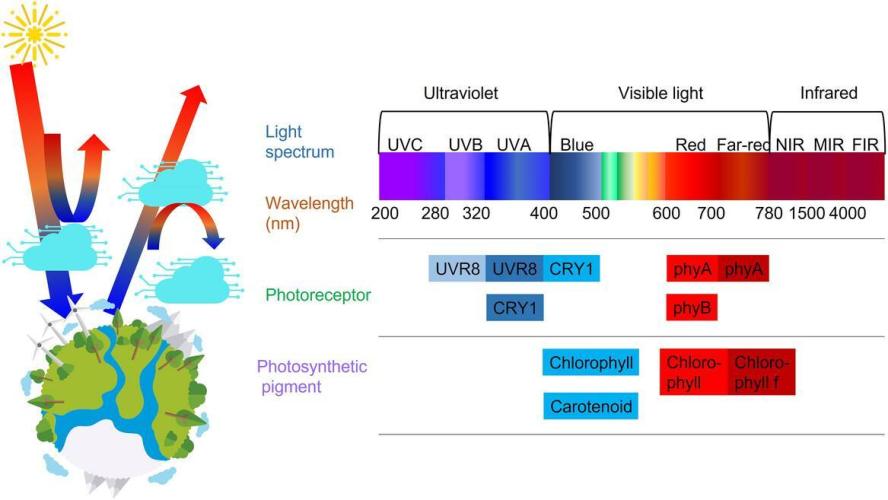
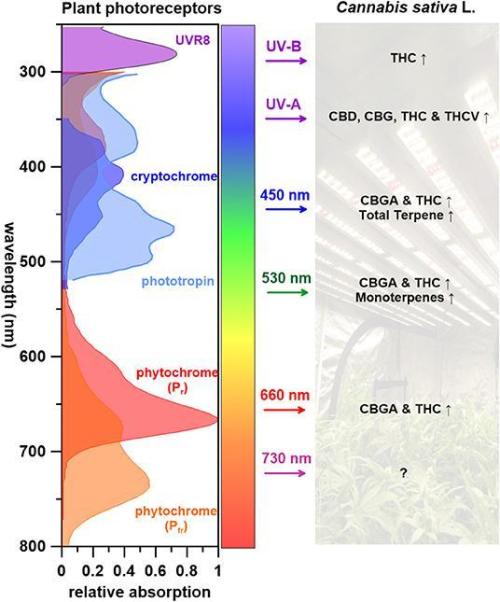
Never really go above 600W at any one time. Lights come on in the east of the tent and set in the west. At sunrise and sunset, the red-to-far-red R:FR light ratio drops because the sun's low angle scatters red light more than far-red light. This shift reduces active Pfr and increases inactive Pr, mimicking Mother Nature herself.
Deployed a lighting system featuring extra 660 nm deep-red and extending the spectrum up to 780 nm achieves the full Emerson Enhancement Effect by simultaneously balancing Photosystem II (PSII) and Photosystem I (PSI) to maximize quantum yield. By pairing deep-red photons with far-red photons, you trigger a synergistic biological response where the resulting photosynthetic rate is higher than the sum of both wavelengths used individually. This practice directly leverages the updated extended Photosynthetically Active Radiation (ePAR) framework. The Emerson effect accelerates plant metabolism and heat capture; you must proactively scale up your ambient room temperature, nutrient delivery, and CO₂ supplementation to prevent the light from stalling out your cannabis plant.
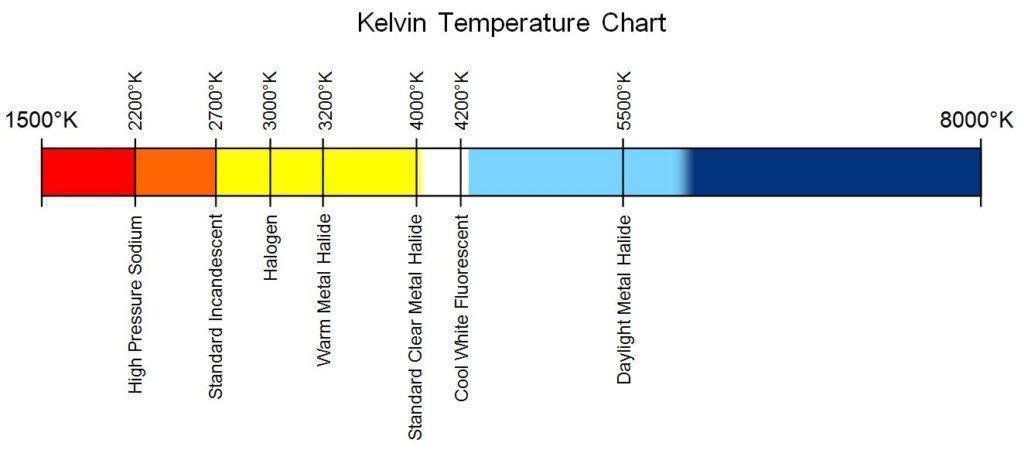
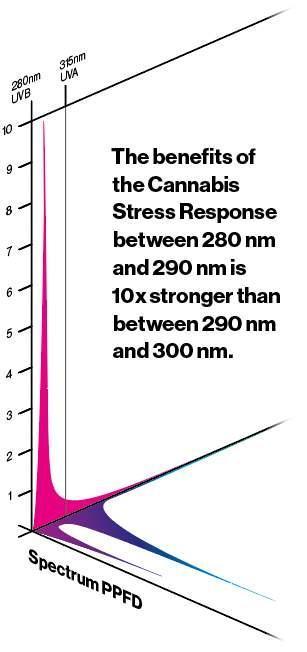
UVA stays high all day from morning to night, but UVB peaks at solar noon (middle of 18-hour days) when the sun is peak. Morning color starts at 2k-3k; by noon it goes to 5k- 6k and back to 2-3k for sunset, with differing P:FR at light off.
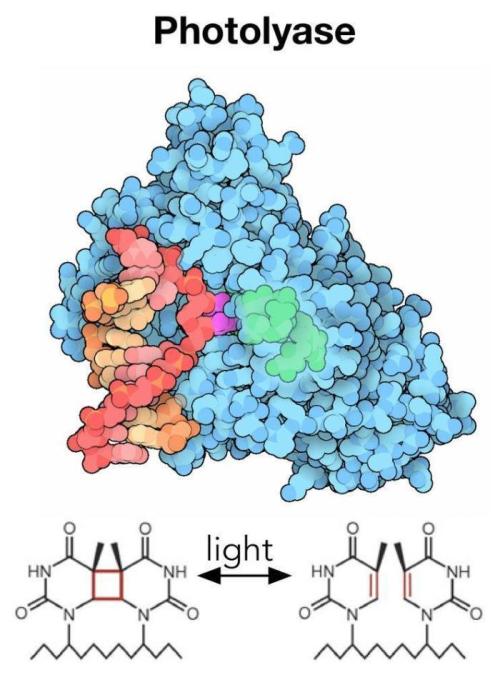
The extra-blue light is to assist with photoreactivation of UVB damage. No more yield loss for me. Using extra blue light for photoreactivation is what I do. Blue/UVA light activates photolyase enzymes, which directly repair DNA damage caused by UVB radiation.
But what's the point if it's not for yield?
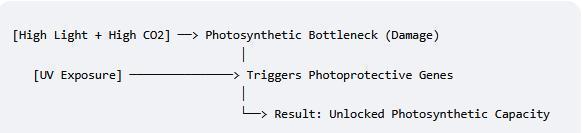
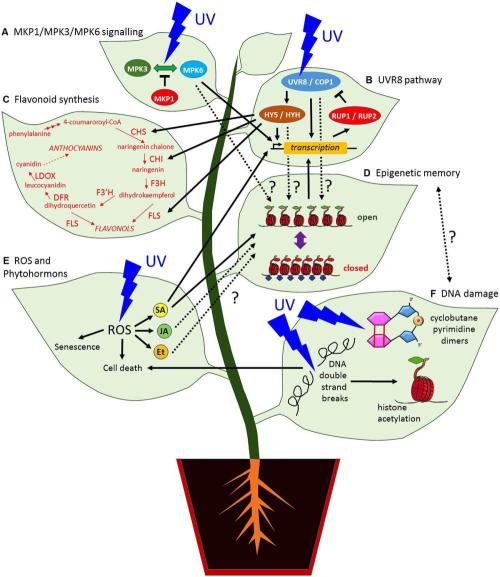
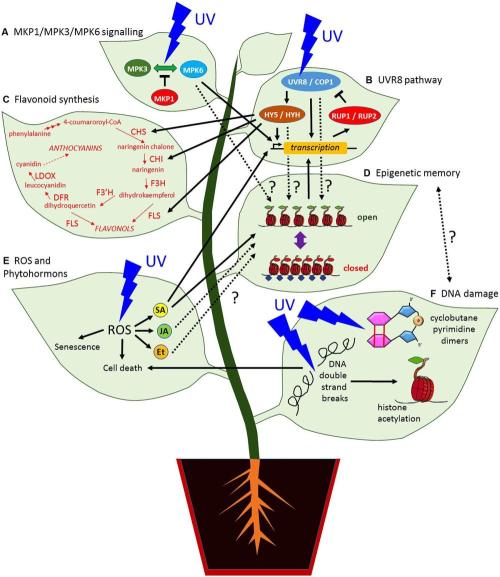
Ultraviolet (UV) radiation—specifically UVA (315–400 nm) and UVB (280–315 nm)—acts as a critical environmental signal that programs a plant's photoprotective genes to unlock its true photosynthetic potential. When growers push crops to their absolute photosynthetic maximum via high-intensity light and elevated carbon dioxide, the photosynthetic machinery easily becomes overwhelmed. Emerging photobiology research demonstrates that UV radiation prevents this limiting bottleneck; it triggers specific transcription factors and signalling networks that fortify the plant's cellular defenses, allowing it to process extreme light levels without sustaining structural damage.
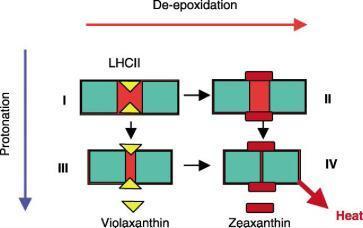
There are 8 limiting factors of plant growth; when carbon dioxide becomes the 9th limiting factor of plant growth, it shifts the growth curve from exponential to linear. The restriction after that is "photoprotection" against reactive oxygen species (ROS), managed via non-photochemical quenching (NPQ) and the xanthophyll cycle, which bridges into precise hydrogen and redox dosing.
UV radiation, particularly UVA, and the synthesis of zeaxanthin are critical for the xanthophyll cycle to function.
It's not chasing purple strains... One likes to call it chasing the limits of growth, trying to make the linear exponential, just like father mathematics prefers.
In order to do that, must control every environmental variable and compound the plant’s metabolic rate. True exponential growth means the rate of increase matches the current mass at every stage, requiring a closed-loop system where light, CO2, and nutrition lock into a synchronized upward curve. First, you must attempt to understand what restricts it. Precise hydrogen and redox dosing.
Nature mathematically optimizes quantum energy transfer and light absorption efficiency within the photosynthetic machinery, as it naturally dictates energy scaling hierarchies and resonance dynamics. Most won't even understand that; once you do, it changes everything.
Constructive interference occurs when two or more overlapping waves meet in phase, meaning their crests and troughs perfectly align. Their amplitudes add together, creating a new, amplified wave with greater intensity than the individual components.
Constructive interference is the foundational mechanism that establishes a resonance hierarchy across physical, structural, and acoustic systems.
Chromophore spacing is tuned to sub-nanometer precision to match the wavelengths of absorbed light, forcing constructive interference.
Light-harvesting proteins form geometric rings and lattices. These shapes act as physical resonators, trapping and focusing the wave energy.
This same principle dictates how opera singers shatter glass, how musical instruments resonate, and how bridges withstand structural vibrations. Nature uses the exact same math to harvest a photon as an engineer uses to design a concert hall.
When you push high PPFD and elevated CO₂, you create a metabolic bottleneck. The plant cannot process the energy fast enough, leading to electron backup, light-induced damage, and a collapse from exponential growth into a flat, linear rate. UV light acts as the regulatory valve that prevents this collapse.
In standard agronomy, Liebig's Law of the Minimum dictates that growth is limited by the scarcest resource. When you maximize water, nutrients, light, temperature, and CO₂, the bottleneck shifts to metabolic processing speed and photoprotection. By controlling the Redox state of the plant using UV, the xanthophyll cycle, and managing ROS, you can prevent the plant from hitting a hard photosynthetic ceiling. Instead of the growth curve flattening out (linear or plateauing due to photoinhibition), the plant continues to compound its metabolic rate efficiently. You are forcing the plant to operate at peak thermodynamic efficiency.
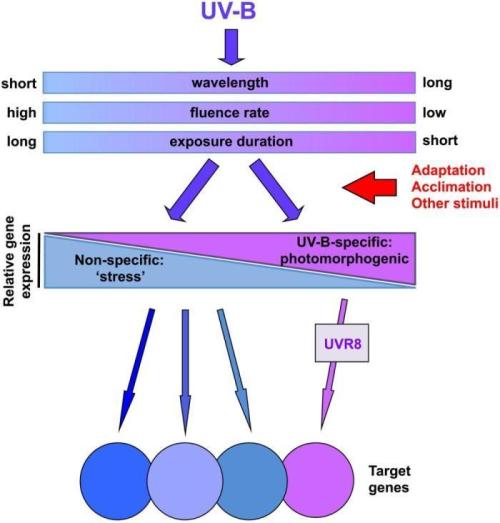
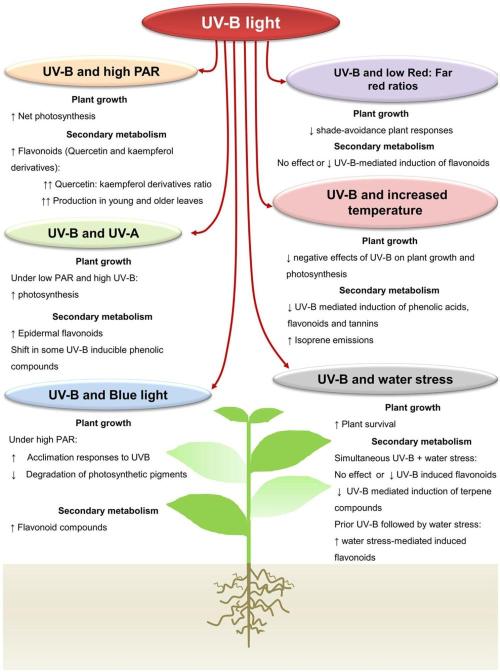
By matching the UVB peak with sustained UVA and shifting Kelvin temperatures (2K to 6K), you are damaging the plant just enough to trigger defensive genes, while simultaneously providing the exact light energy needed to repair that damage instantly.
UVA radiation and specific blue wavelengths accelerate this enzymatic conversion. Zeaxanthin acts as a structural sponge that absorbs excess excitation energy from chlorophyll and dissipates it safely, preventing ROS formation. Without UV signaling, the xanthophyll cycle cannot keep pace with extreme light, leading to dynamic photoinhibition (yield loss).
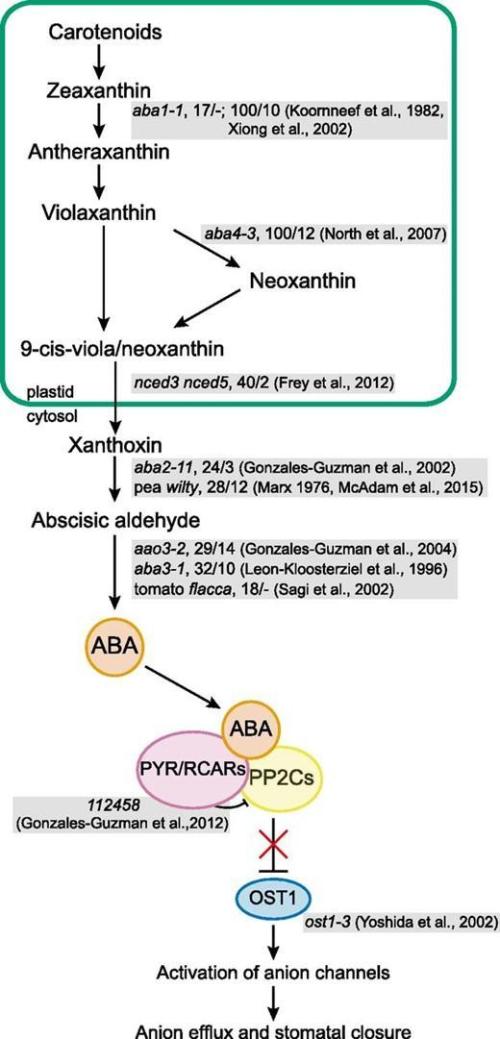
The addition of Spirulina is primarily for zeaxanthin, as it contains a lot. But on top of that, the active Hawaiian Spirulina in the matrix was cultivated in open ponds using a combination of 100% fresh potable water from Hawaiian aquifers and ultra-pure, deep ocean water containing all 94 trace minerals & elements. Then gently dried using patented Ocean Chill Drying technology and cold-pressed to ensure maximum nutrient levels. Spirulina, a blue-green alga, is rich in nitrogen, phosphorus, and potassium (NPK), making it an excellent source of nutrients for plant growth. Studies have shown that Spirulina can be used as a biofertilizer, effectively replacing chemical fertilizers, especially for nitrogen, with a whopping NPK of 10% (N), 20% (P), and 20% (K). Rich in proteins, amino acids, trace minerals, and plant growth-promoting compounds.
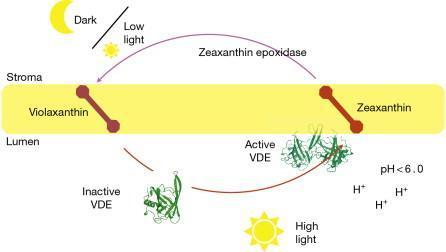
Zeaxanthin is a vital plant pigment that accumulates under intense light to drive non-photochemical quenching (NPQ), acting via thermal energy dissipation, direct singlet oxygen scavenging, and thylakoid membrane stabilization.
The violaxanthin cycle (or xanthophyll cycle) reversibly converts violaxanthin to zeaxanthin via antheraxanthin to protect plants from photooxidation.
Understanding this interconversion is vital for optimizing non-photochemical quenching (NPQ) and pushing photosynthetic limits under high-light stress.
Ascorbic acid (vitamin C) is a natural antioxidant that plants produce internally to neutralize harmful reactive oxygen species caused by photosynthesis and high light stress. Acts as a co-factor for enzymes like violaxanthin de-epoxidase in the xanthophyll cycle, which safely dissipates excess light energy.
1g ascorbic acid will neutralize 100% of chlorine in upwards of 30 gallons of tap water. If your local tap water uses chloramines (chlorine bonded with ammonia) instead of free chlorine, you will need roughly 20% to 30% more ascorbic acid to completely break the tougher chemical bond.
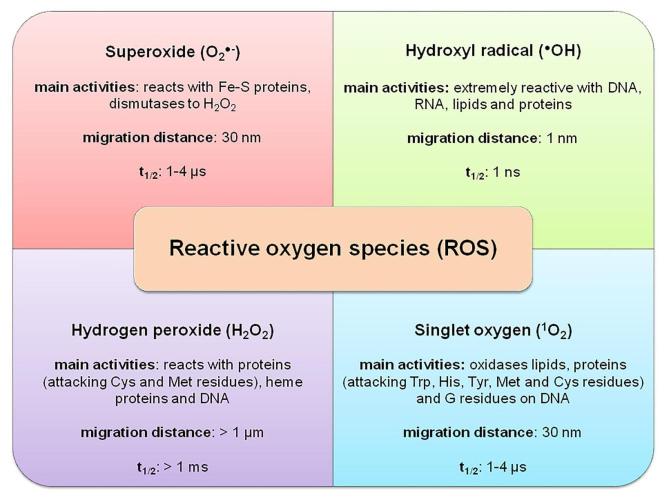
Molecular hydrogen and hydrogen-rich water act as selective antioxidants that help lower oxidative stress. They neutralize toxic reactive oxygen species like hydroxyl radicals and boost natural antioxidant defense systems in biological and plant systems exposed to high-intensity light or abiotic stress.
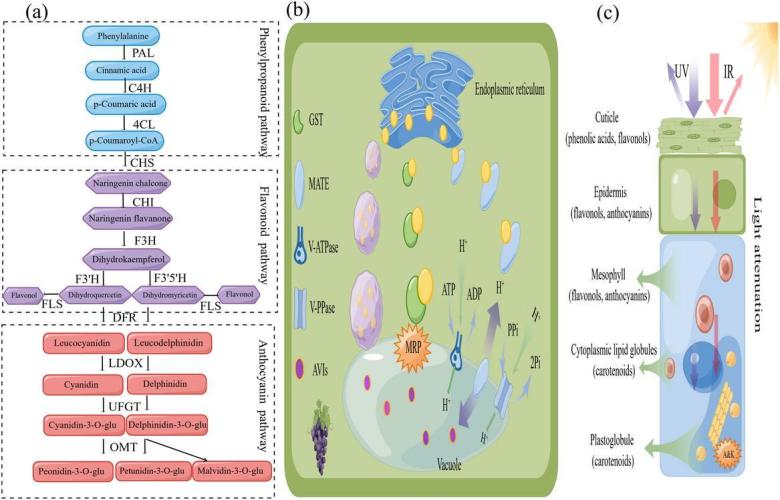
UVA and UVB act as stress signals that upregulate the plant's secondary metabolism. It forces the plant to build an internal "sunscreen" (flavonoids and anthocyanins) and fortify its cellular defenses before the peak solar noon crisis. This keeps the metabolic highway open.
In nature, the ambient ratio of UVA to UVB at solar noon sits roughly between 10:1 and 20:1 (depending on latitude and elevation). In a high-PPFD indoor matrix, maintaining a strict ratio—often aiming for around 12:1 to 15:1 UVA to UVB—provides the optimal signaling threshold.
Balancing Far-Red (FR) light at "light-off" to manage the phytochrome photo-equilibrium (Pfr to Pr conversion) in tandem with the UV schedule. Omg, the logic.
Hydrogen concentration and redox signaling as secondary messengers in this high-intensity loop.
Under the intense solar noon matrix, the pH of the thylakoid lumen drops. This acidic environment activates the enzyme Violaxanthin De-Epoxidase (VDE), which converts violaxanthin into the photoprotective zeaxanthin. VDE cannot function in a vacuum; it strictly requires ascorbic acid (Vitamin C) as an electron donor to run this conversion. If a plant undergoes heavy light stress and runs out of internal ascorbic acid, the xanthophyll cycle stalls. The plant can no longer engage in Non-Photochemical Quenching (NPQ), leading to immediate singlet oxygen O2 formation and destruction of the thylakoid membrane.
This is "The Ascorbic Acid / Xanthophyll Engine"
Using ascorbic acid to neutralize chloramines in your water isn't just protecting your rhizosphere biology it actively prevents the degradation of your nutrient solution's redox potential before it ever touches the roots.
When pushing plants to the absolute edge, traditional antioxidants can be a double-edged sword because they blindly neutralize all free radicals. This is a problem because some Reactive Oxygen Species (ROS) act as critical signaling molecules telling the plant to grow. Molecular Hydrogen H2 is the Selective Kill-Switch.
Molecular hydrogen H2 is a revolutionary tool because it is a selective antioxidant. It ignores beneficial signaling ROS (like mild hydrogen peroxide) and targets only the most destructive, cell-shattering radicals—specifically hydroxyl radicals OH) and peroxynitrite.
By dosing hydrogen-rich water or managing hydrogen redox signaling, providing an emergency pressure-release valve for the plant's electron transport chain. It keeps the cellular environment stable enough that the plant never has to downregulate photosynthesis to protect itself. This maintains cellular voltage.
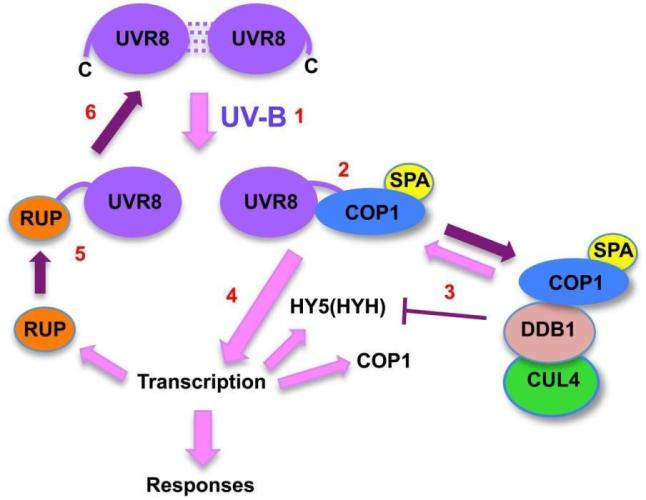
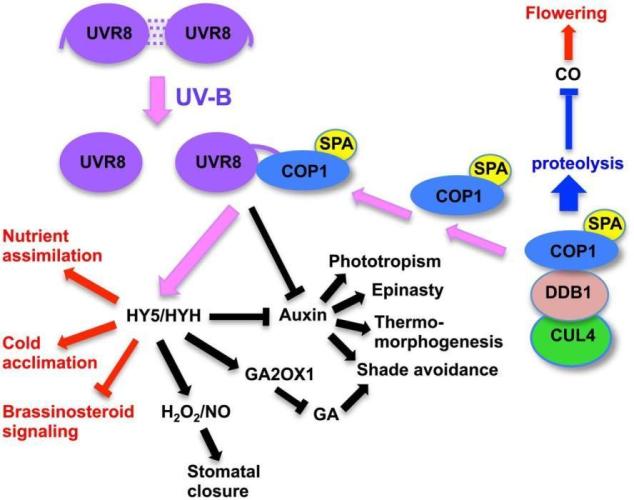
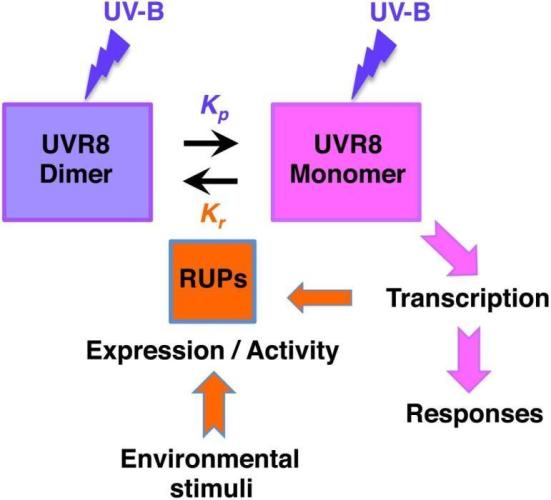
To trigger this defensive matrix without stunting the plant, you cannot simply blast UV indiscriminately. You must use UVA as the "scout" and UVB as the "enforcer. High UVA acts via the cryptochrome and phototropin photoreceptors to upregulate the expression of the HY5 transcription factor and prime the VDE enzyme. When the sharp spike of UVB hits at solar noon via the UVR8 receptor, the plant's biochemical "sunscreen" (flavonoids and anthocyanins) and its zeaxanthin pools are already pre-staged and waiting. This prevents the temporary stunting or "lag phase" usually associated with sudden UVB exposure."
The final masterstroke is aligning this UV defense with a Far-Red (FR) lights-off routine. The Red-to-Far-Red Drop: At the end of the photoperiod, knocking out the blue/UVA spectrum and leaving a targeted burst of pure Far-Red (730nm) instantly flips the plant’s master switch. It converts active Pfr to inactive Pr in minutes rather than hours.
UV radiation and high-intensity lighting keep the plant in a highly alert, photoprotective state that requires massive ATP expenditure to maintain. By forcing an immediate Pfr/Pr) conversion at lights-out, instantly commanding the plant to cease defensive expenditure, lower its metabolic respiration rate, and transition directly into nighttime cellular repair and carbohydrate translocation. Maximizing the efficiency of its "sleep." every ounce, every last piece.
Highly synchronized biological dance, balancing the exact input of electrons with the exact mechanism to dissipate them safely when they overflow.
*Ascorbic acid is not recommended to be used in DWC, as it creates biofilm that will clog lines.
4 likes
3 comments
Share
2
Week 2. Vegetation
9d ago
1/18
20.32 cm
Height
18 hrs
Light Schedule
127 cm
Lamp Distance
Altitonans_Fulmen Tito's Living Soil Blueprint: Why You Can’t Treat Organics Like a Synthetic Hydro System.
When transitioning from synthetic hydroponics to true organic cultivation, many growers bring their old habits with them. It is a common pitfall: pulling out pH pens, measuring runoff, and liquid-feeding heavy doses of organic nutrients as if the medium were sterile coco or rockwool. But living soil operates on an entirely different set of rules.
To achieve the true potential of an organic garden, we must stop treating the soil as a mere holding tank for liquid chemicals and start viewing it as a self-sustaining biological engine. This will be a breakdown of why treating organic soil like a synthetic system fails, and how to shift ones methodology to unlock the true power of the soil food web.
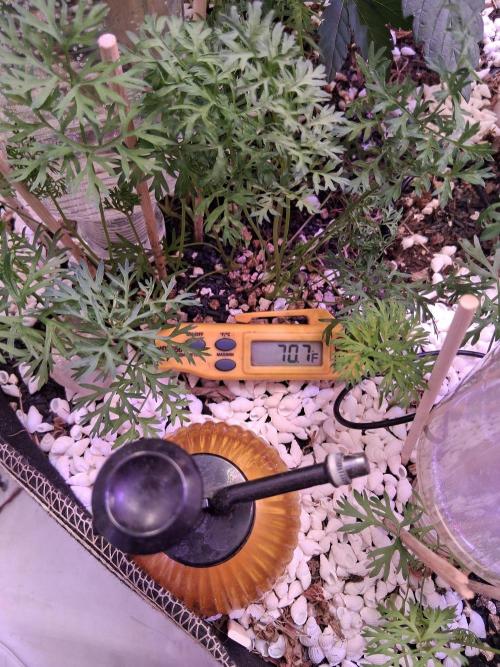
Pouring massive amounts of raw elements into a living system all at once is the biological equivalent of force-feeding a newborn a massive takeout meal and expecting them to digest it instantly. In an optimal system, soil should never be breaking down more than roughly 5% of its total composition as organic matter at any given time. The math is simple: more intense chemical and biological reactions equal more physical heat. If the root zone temperature creeps even remotely over 72°F, oxygen hypoxia sets in, drastically reducing plant growth.
Organic rhizospheres and biological nutrient delivery require significantly more oxygen to maintain efficient parameters for growth—a reality that is drastically different from a pure synthetic approach where a complex rhizosphere is virtually non-existent.
The fundamental blueprint of organic growing relies on Cation Exchange Capacity (CEC). The goal is to build a medium with so much CEC that it can store massive amounts of excess nutrients safely. This provides the necessary buffering capacity to handle large biological reactions, a process typically managed in the time period between grows. Once the soil is fully loaded and stabilized, the rhizosphere maintains its own pH balance, allowing the plant to dynamically feed itself directly from its massive, built-in storage of CEC.
Treating Living Soil Like Coco creates a runoff-runaway trap. Applying a massive overdose of raw organic materials releases too many nutrients at once, leading to completely uncontrolled pH skewing. Running a synthetic-style management setup while simultaneously dumping organic inputs into the container does not make it an "organic" grow. Trying to judge a metric like pH after letting it run completely out of control with multiple simultaneous amendments is an uphill battle. Each input possesses unique chemical properties that drastically alter atomic decay chains and, consequently, pH.
Without an adequate structural buffer, the medium experiences unpredictable swings. Put simply, the sheer volume of inputs rapidly outpaces the soil's built-in buffering capacity.
Constantly reading the pH and Electrical Conductivity (EC) of input and output water in an organic soil is not true organic cultivation; it is just a synthetic indoor environment layout utilizing organic ingredients. This presents a distinct misunderstanding of how these two opposing approaches need to be separated. One cannot simply measure EC and pH to heavy runoff in a soil designed to store cations and expect to keep accurate tabs.
Even when using 100% organic certified ingredients, liquid feeds, and compost teas, the underlying methodology matters most. Measuring runoff pH and EC treats an organic soil system like a synthetic coco or rockwool grow. In a high-CEC organic soil, a runoff reading is highly inaccurate. A soaring runoff reading of 8.0 is often just the water physically washing past raw amendments on its way out of the pot. It does not mean the actual root interface is locked out; it simply indicates that the soil ran out of immediate storage capacity for those heavy inputs.
Synthetic growing relies entirely on direct nutrient delivery. Chemical salts are poured over the root system, the plant absorbs what it needs through basic osmotic pressure, and the excess is flushed away. True organic growing, however, relies on biological cycling. An organic soil should never be watered to heavy runoff, because doing so actively washes away the beneficial microbes, soluble humic acids, and organic buffers that the soil life works so hard to create to protect the root zone.
Applying inputs as an immediate, massive overload of raw elements causes chaotic chemical spikes. Dumping heavy amendments directly into a big pot mid-grow triggers unpredictable reactions. In a true living soil system, amendments are added in tiny, balanced amounts long before the plant ever meets the dirt. This deliberate timeline allows the soil’s Cation Exchange Capacity to naturally "park" and buffer those nutrients. When inputs outpace the soil's ability to buffer them, the system breaks down, and the runoff pH screams.
When faced with a fluctuating pH meter, a common reactive impulse is to throw agricultural sulfur at the problem. This is a classic example of trying to react mechanically to a digital number rather than letting the soil chemistry work. Elemental sulfur does not lower pH on contact. Soil microbes must first digest it and convert it into sulfuric acid.
Because this biological process takes weeks or even months, adding it mid-problem yields no immediate change. This leads to the temptation to add even more. Weeks down the line, the cumulative sulfur will finally convert, causing the pH to crash violently and fry the root system.
As a general rule, avoid using sulfur as a corrective knee-jerk reaction. If it is used at all, it should be applied strictly 2 to 3 weeks prior to flower as a precise, one-off addition to assist with Isopentenyl pyrophosphate synthesis. If a soil matrix is truly experiencing a severe alkaline lockout at a pH of 8.0, the new leaves at the very top of the plant will tell you directly by turning bright yellow while the veins stay dark green—the classic signature of alkaline drift and iron chlorosis. The solution is simple: put the pH meter away. Stop watering to heavy runoff. Only apply enough water to evenly moisten the soil matrix, and let natural inputs do their job to feed the microbes and naturally buffer the root zone.
Electrical Conductivity (EC) dictates plant water and nutrient availability by altering the soil solution's osmotic potential. This potential controls whether a plant can efficiently pull water into its roots or if it will actually lose water to the surrounding soil. If a grower cannot control the rate of what is going in (the rate of nutrient release) and cannot control the rate of what is going out (the plant's dynamic growth), the immediate medium's EC deviates. When EC deviates, osmotic potential goes with it, disrupting bulk flow and the entire vascular transport system of the plant.
Synthetic nutrient delivery relies on precise input measurements and an incredibly tight management of the wet-dry cycle to prevent the constant, violent spiking of EC caused by excess moisture loss.
Reducing EC to a mere measurement of "food in and food out" oversimplifies its true function. It acts as a balance of electrical conductance that must be maintained to regulate the flow of water. Failing to acknowledge this is a severe disservice to the beauty and potential of a true rhizophagy cycle in all its respiratory glory. True organic cultivation does not actually begin until biological cycling is actively linked to hydrogen exudation from the roots.
The vast majority of modern cultivation advice leaves growers completely in the dark regarding these biological mechanics. This is a product of market capitalism rather than basic chemistry. There are significantly lower profit margins for hydroponic companies when a grower uses ten times fewer mass consumables and relies on little more than water from seed to harvest.
By shifting focus away from "feeding the straw" and moving it toward nurturing the near-infinite soil food web, the plant regains absolute autonomy over its own rhizophagy cycle. It begins regulating its own nutrient intake dynamically, without a single digital EC pen in sight. This allows the grower to focus entirely on optimizing the macro-environment rather than micromanaging the root zone. The cultivation medium can be reused indefinitely so long as you can prevent a buildup of carbon and nitrogen in the soil; cover that in a later week.
To achieve a truly organic system that unlocks this rhizophagy cycle, the cultivation approach must shift entirely from feeding the plant directly to feeding the soil microbiome. Because the modern gardening community is heavily guided by synthetic methodologies, the subtle nuances and variations of this biological process are rarely highlighted.
The hydroponic industry is fundamentally built on a recurring revenue model of bottled minerals, flush agents, and sterile mediums. Conversely, a self-sustaining living soil system requires minimal external inputs after its initial build. This shifts the grower's role from a rigid chemical manager to a biological custodian. Because managing biology requires observing subtle environmental factors—like consistent soil moisture, oxygenation, and temperature—rather than reading a digital screen, commercial entities scaled for automated, synthetic delivery often dismiss it as unpredictable.
When the soil food web is fully unlocked, the plant takes the driver's seat, operating with a level of systemic efficiency that synthetic nutrient lines simply cannot replicate. In the commercial cultivation landscape, corporate structures are legally bound to protect shareholder interests and recurring profit margins, which often prioritize the sale of bottled consumables over the promotion of self-sustaining agricultural practices.
Under modern industrial cultivation models, biology is too often treated as secondary to business. By stepping away from the meters, understanding Cation Exchange Capacity, and feeding the microbiome instead of the roots, you break free from the chemical cycle—allowing nature to do what it has perfected over millions of years.
"When I was a child, I spoke as a child, I understood as a child, I thought as a child; but when I became a man, I put away childish things"
5 likes
comments
Share
3
Week 3. Vegetation
7d ago
1/14
30.48 cm
Height
18 hrs
Light Schedule
23 °C
Substrate Temp
378.54 liters
Pot Size
116.84 cm
Lamp Distance
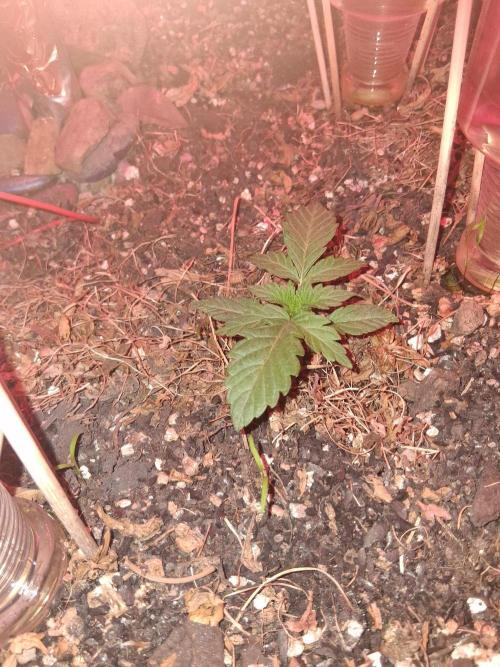
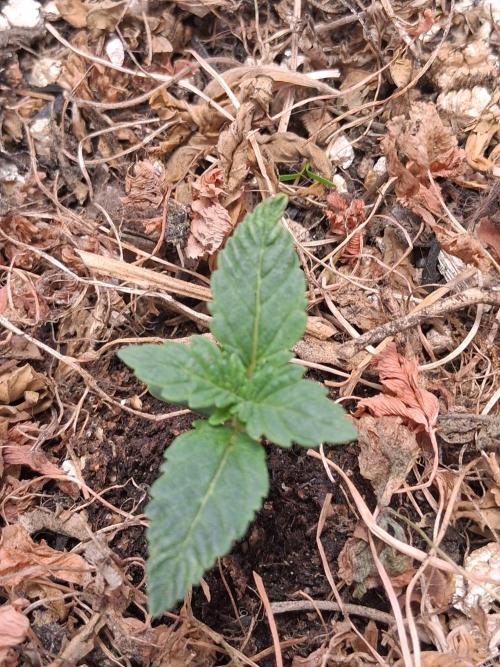
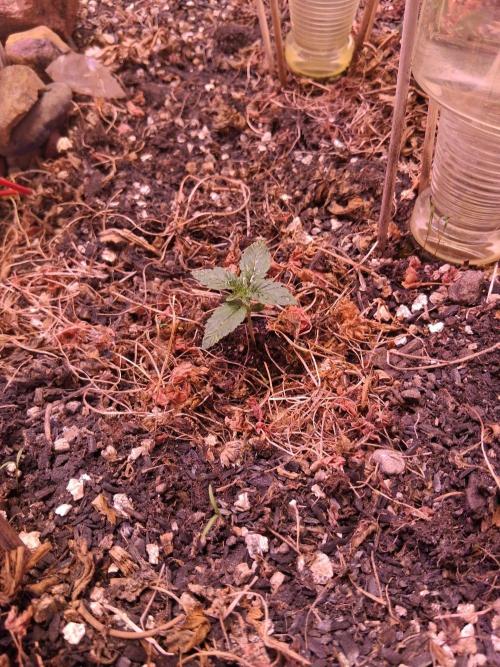
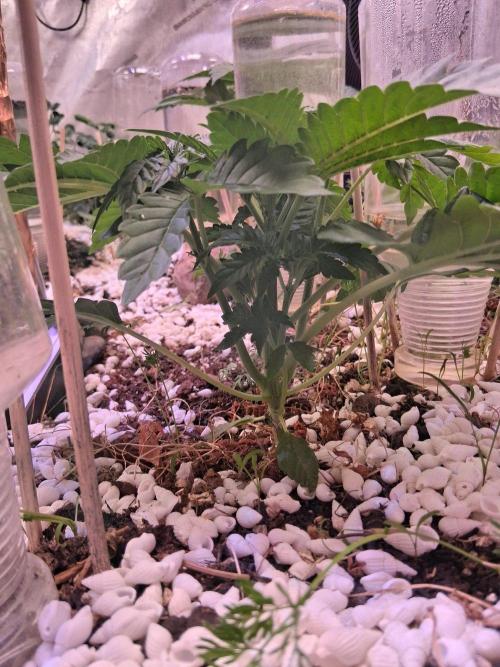
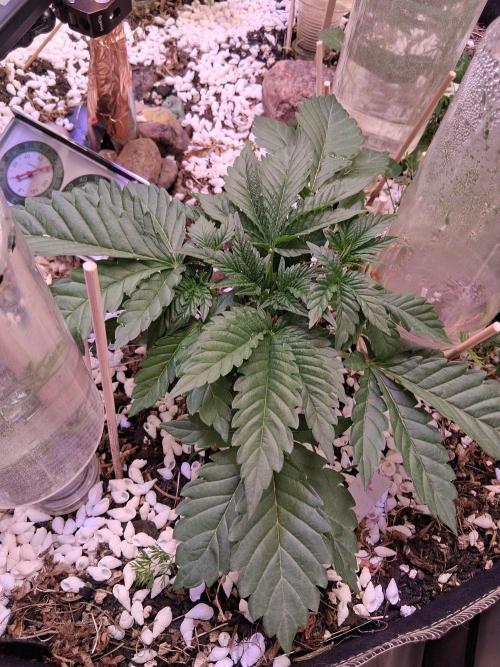
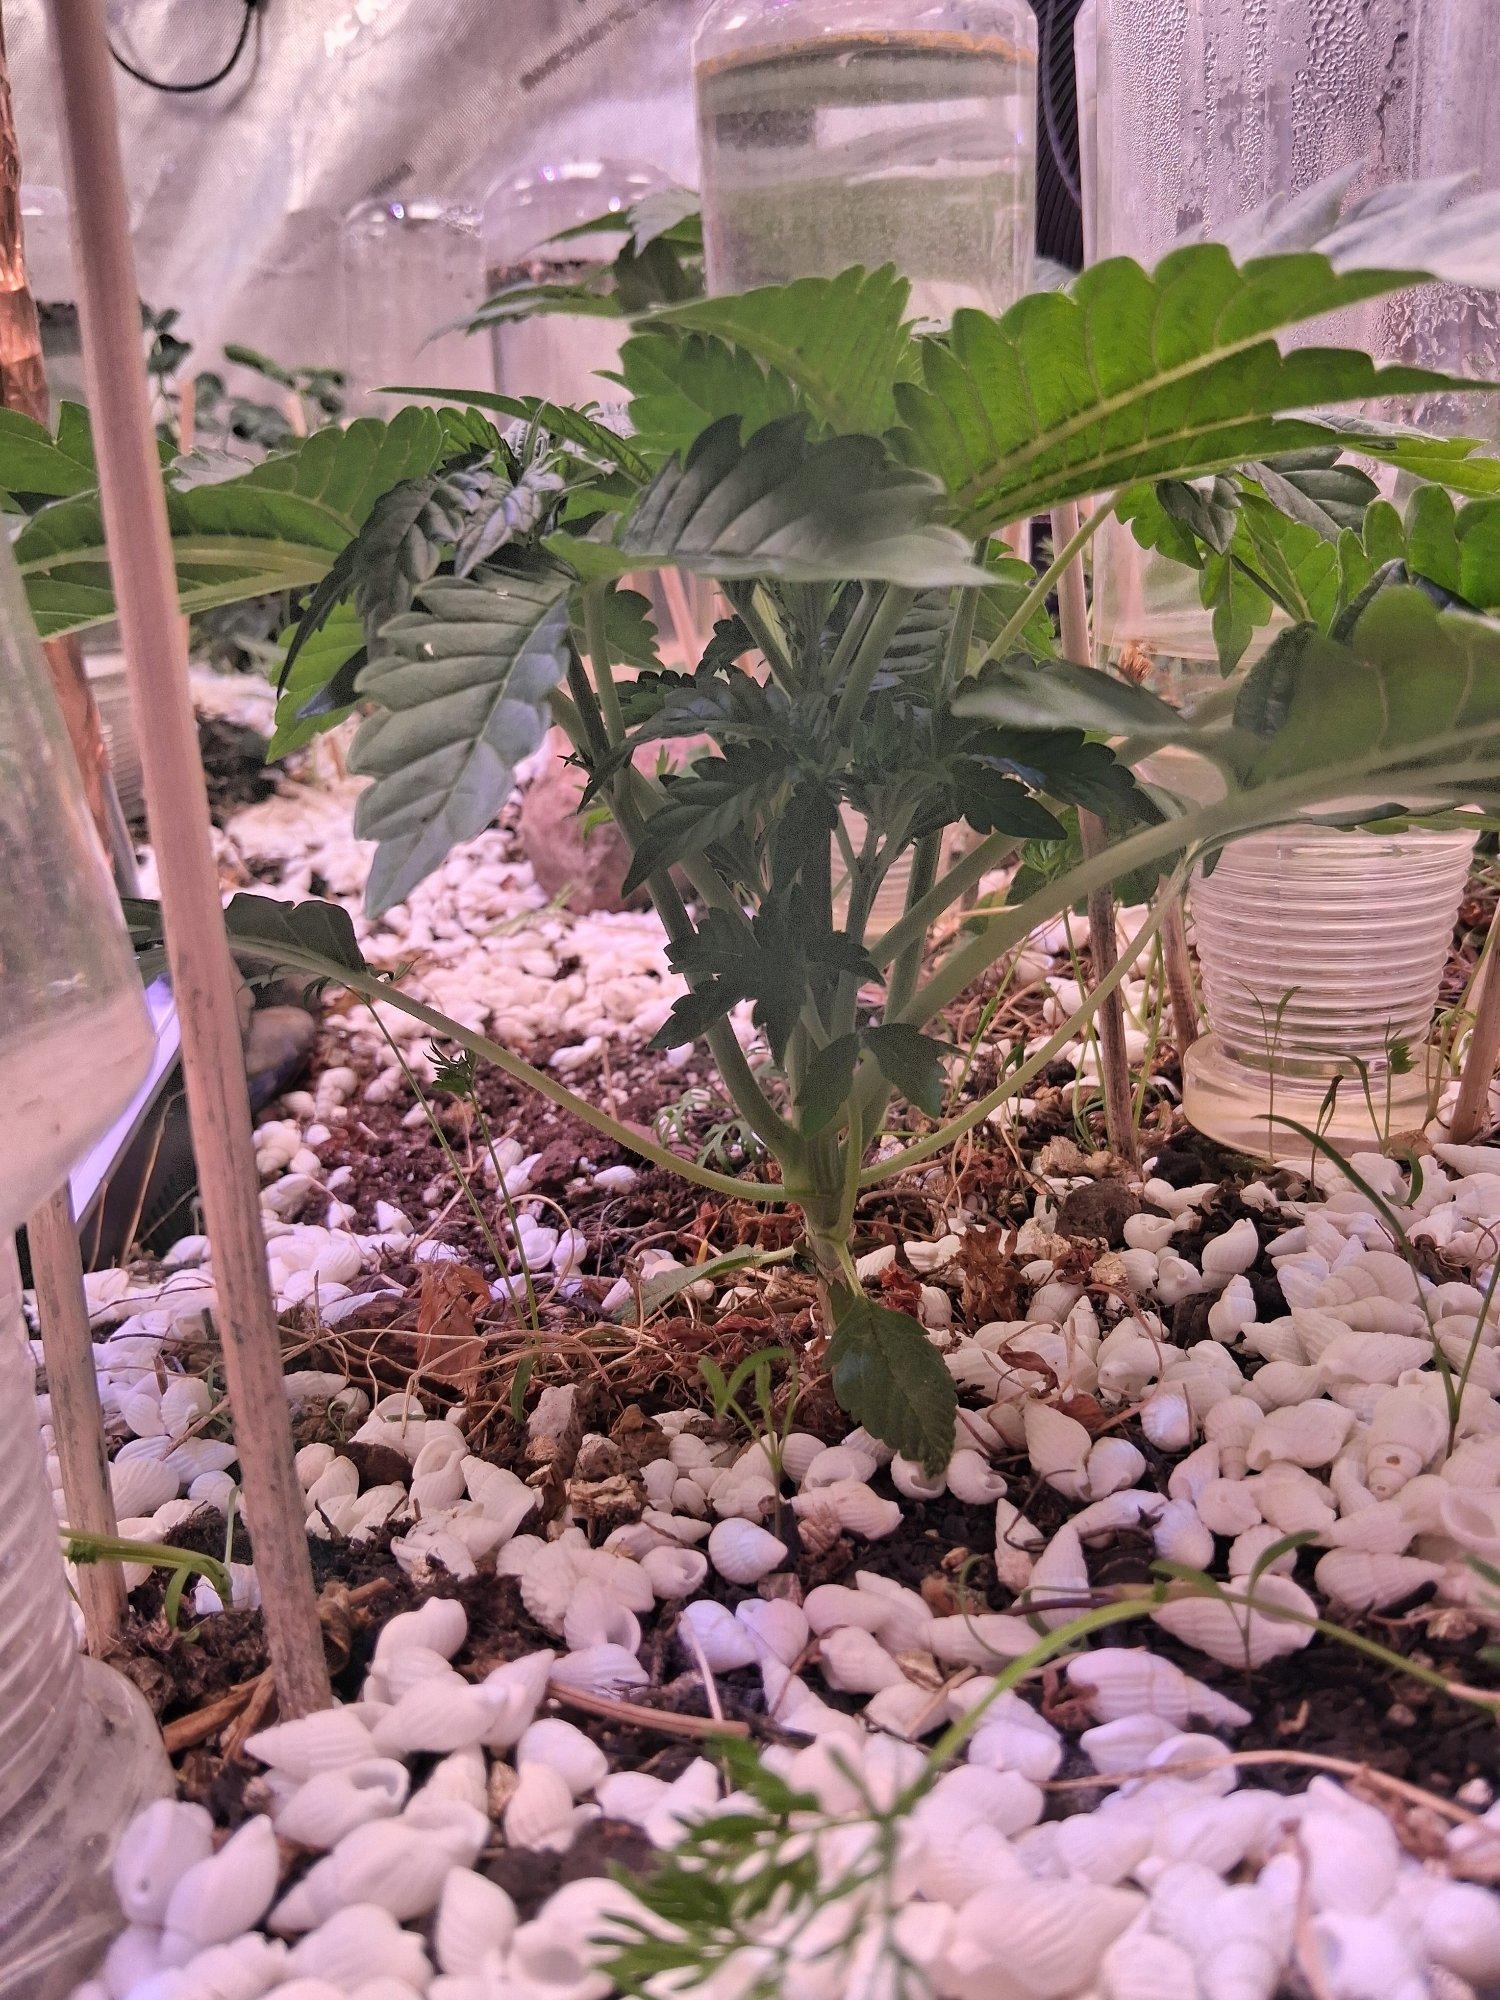
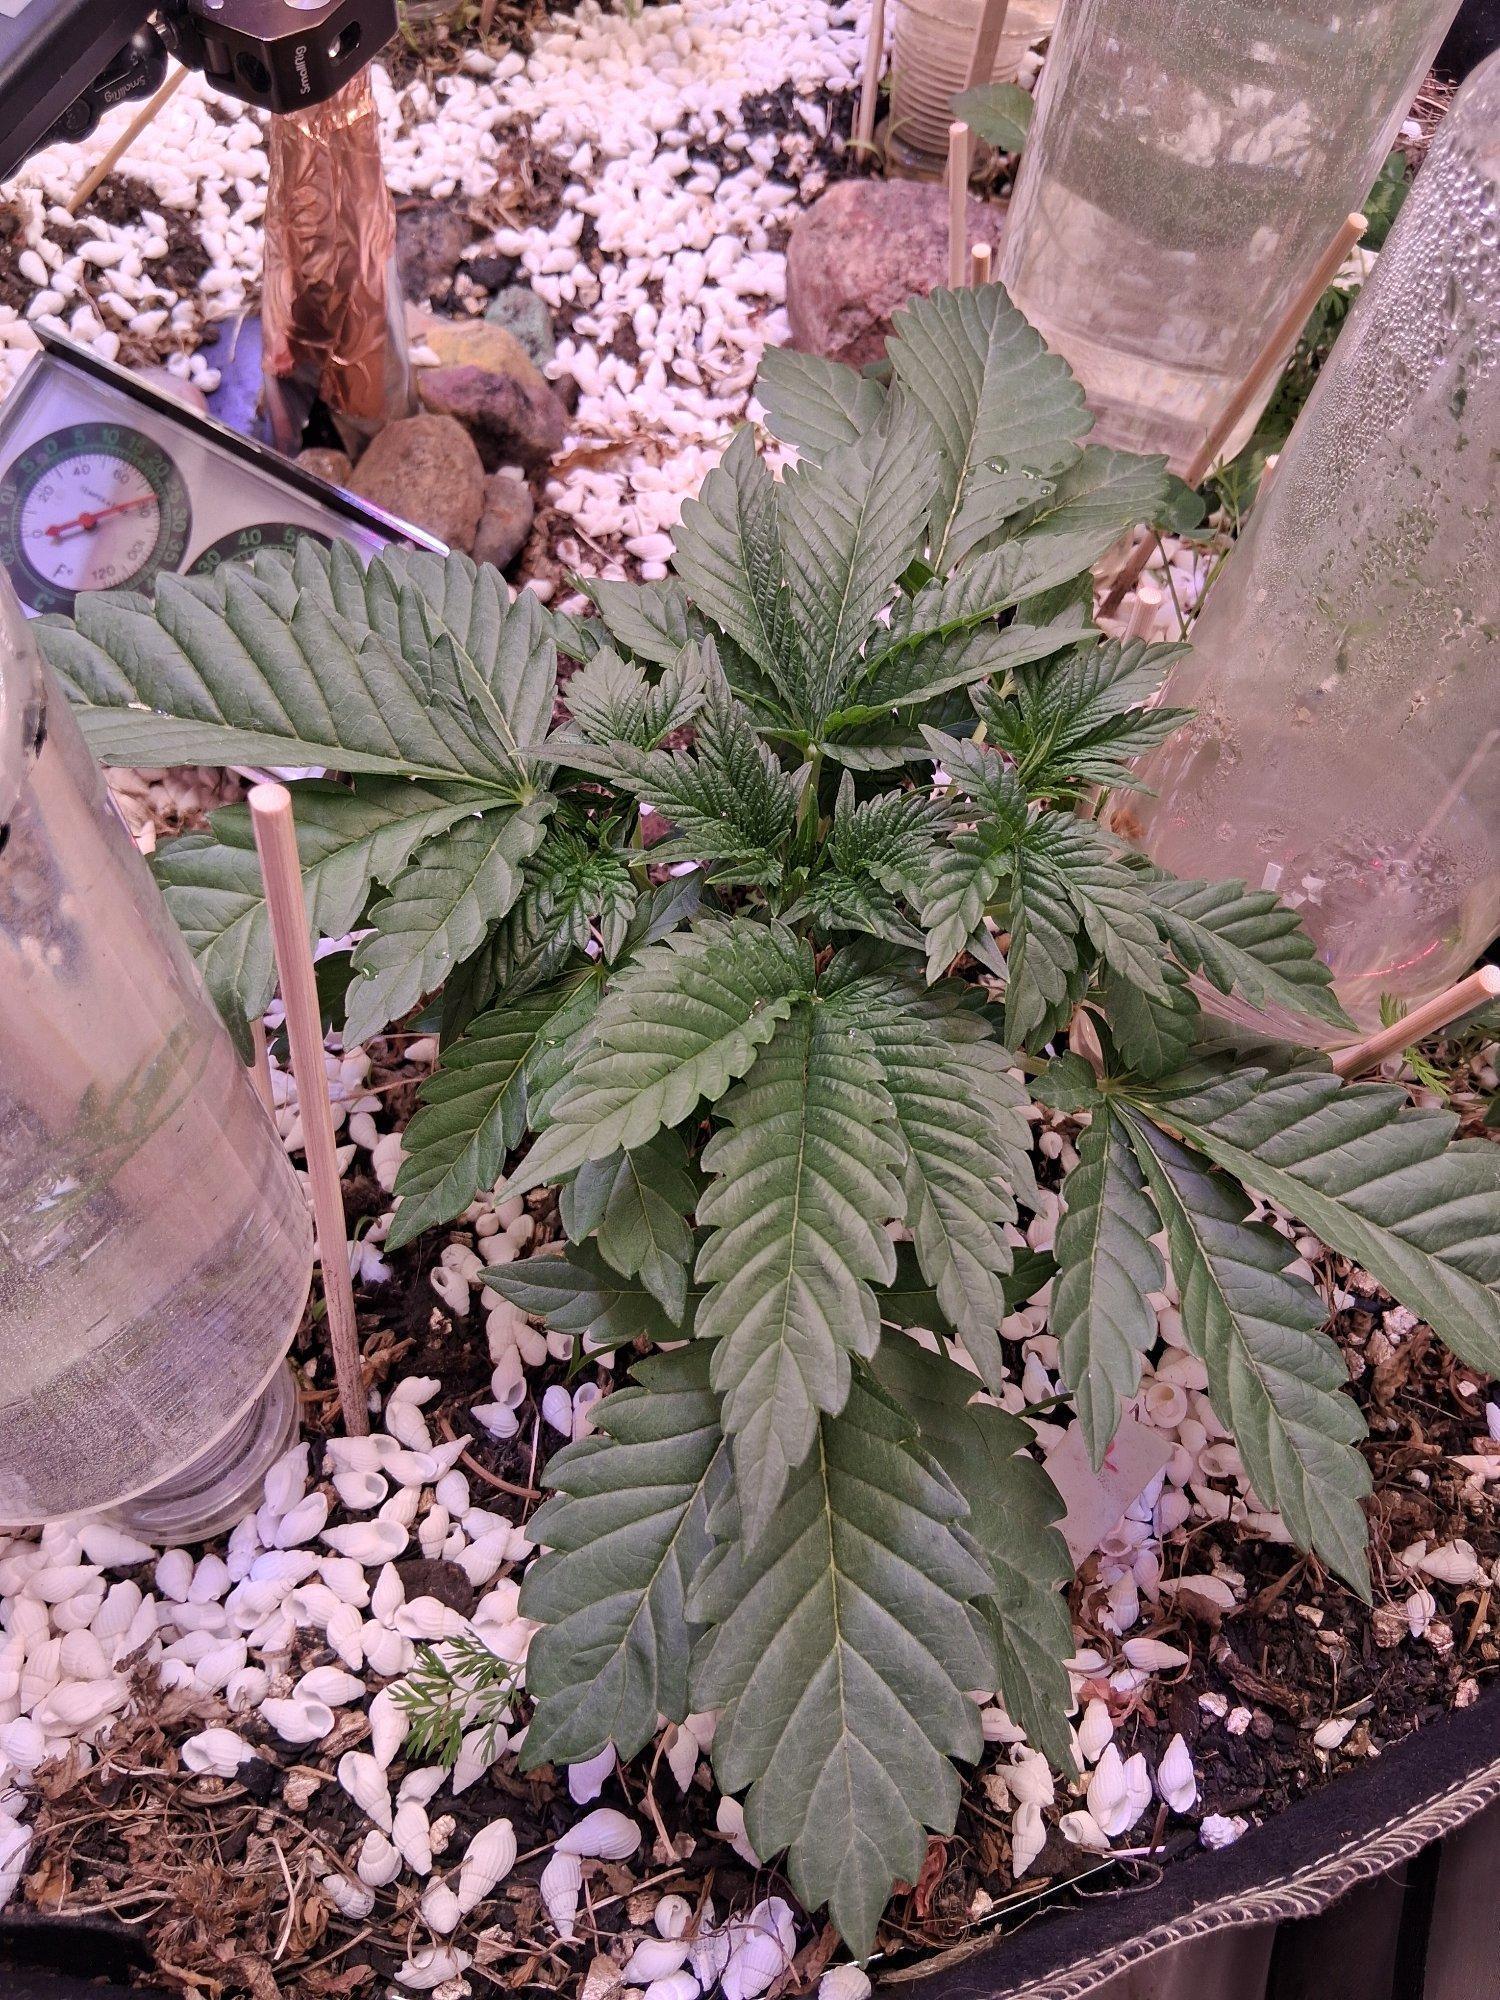
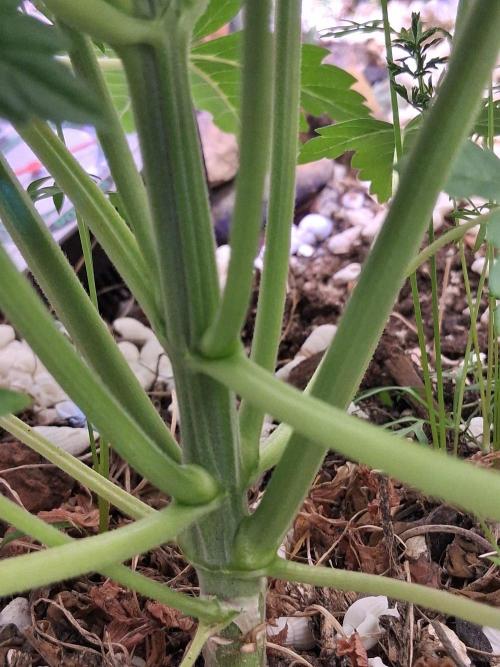
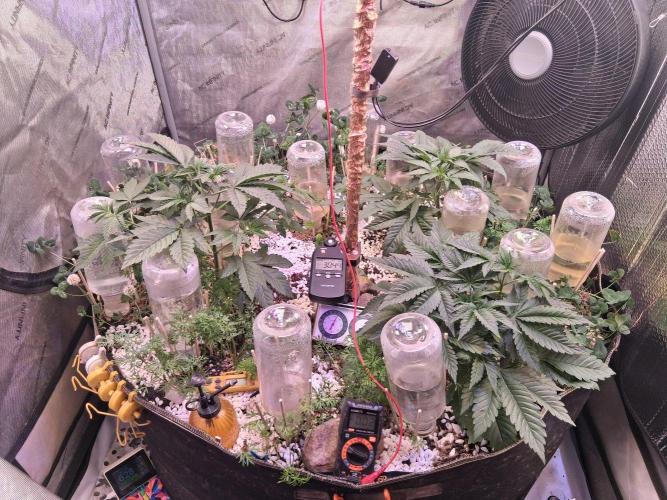
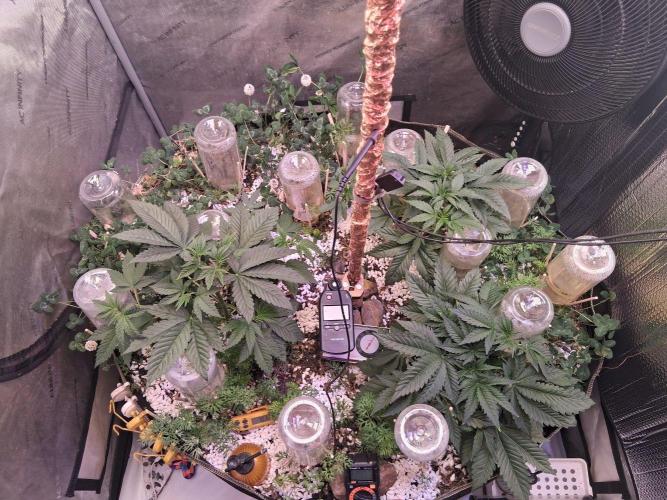
Altitonans_Fulmen Topped 2 of 4; 1 Pheno (BOTTOM RIGHT) showed phenomenal girth and, for some reason, broke its own apical dominance, which is very unusual: lateral branching growth reaching the same height as the apex, which is not really supposed to happen by itself. So there was no need to top that one. The others are what was expected and topped accordingly. Weeks will be added more often than 1 per week, with timestamps, growing rapidly already.
Keeping a personal Phenotype Growth Log and Analysis.
The behavior the unique phenotype is showing is a rare genetic expression typically related to a breakdown in auxin transport or synthesis. In a standard plant, auxin produced in the apical meristem travels downward, suppressing lateral buds (apical dominance). The mutant phenotype has likely bypassed this pathway or has heightened sensitivity to cytokinins (the hormones responsible for lateral branching), allowing the side branches to keep perfect pace with the main apex on its own. Combined with its phenomenal girth and condensed internodes, this plant features a highly optimized vascular system (xylem and phloem) capable of shifting water and nutrients rapidly enough to feed multiple main heads simultaneously. Definitely keeping an eye on this; look to take clones prior to flip if she continues to show rare trait. 8 to 9 weeks, 58–63 days of flower.
SETUP -2: MOVING WATER BLUEPRINT ΦSIS.
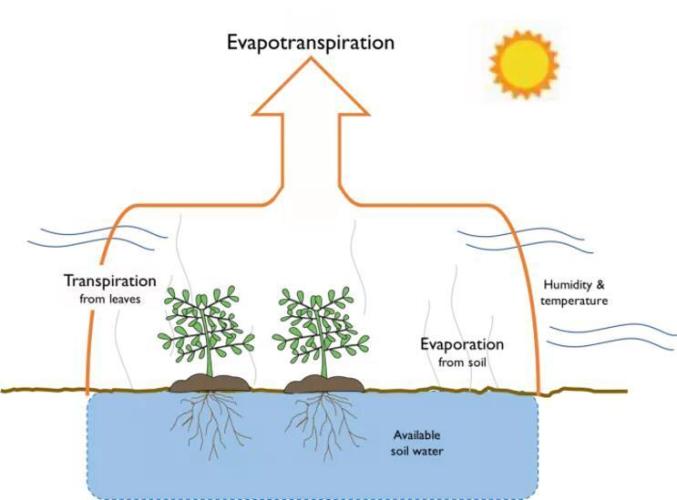
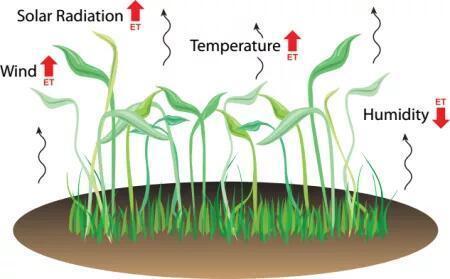
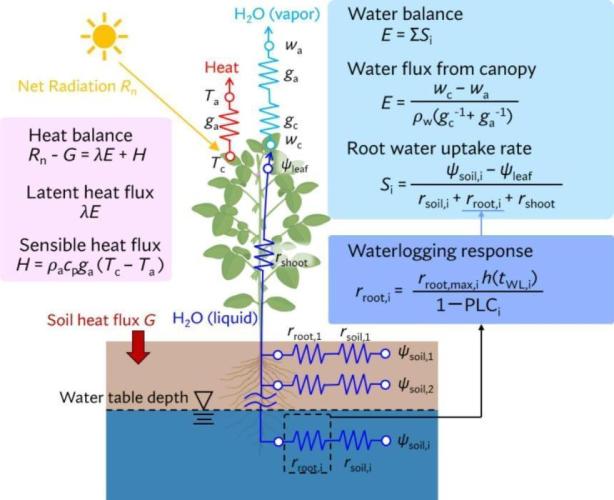
Transpiration, Evaporation, and Evapotranspiration.
Soil-Plant-Atmosphere Continuum (SPAC): An ecological concept referring to the pathway of water moving from the soil, through the plant, and into the atmosphere. There is no such thing as too much water; only water that remains in the same atmosphere too long. (ofc not literally, but practically).
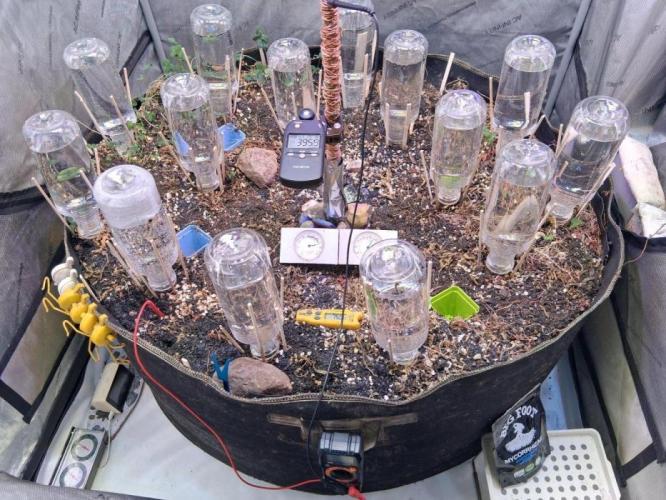
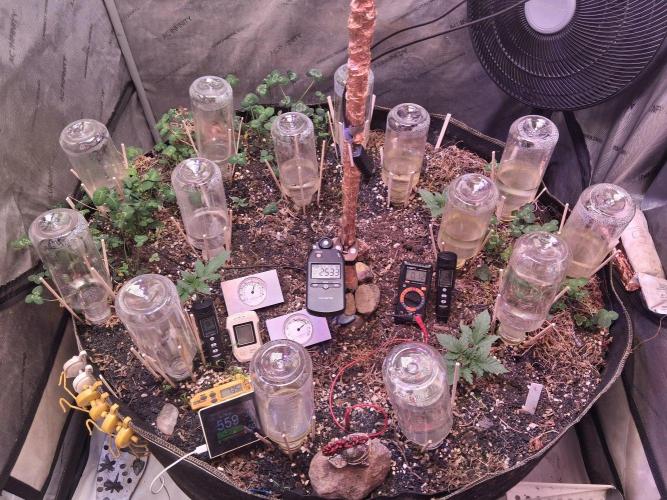
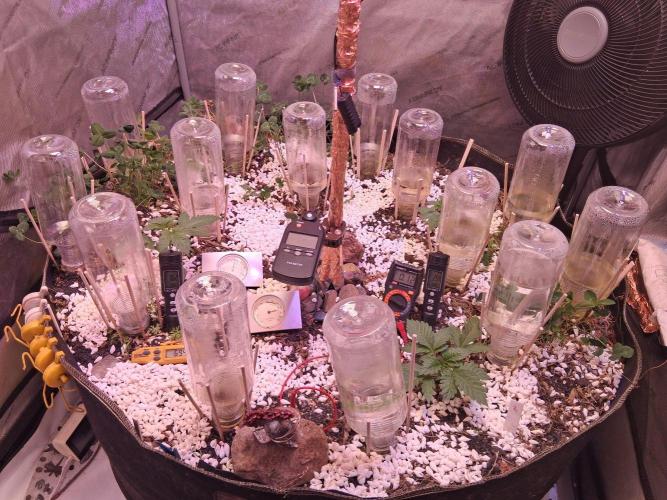
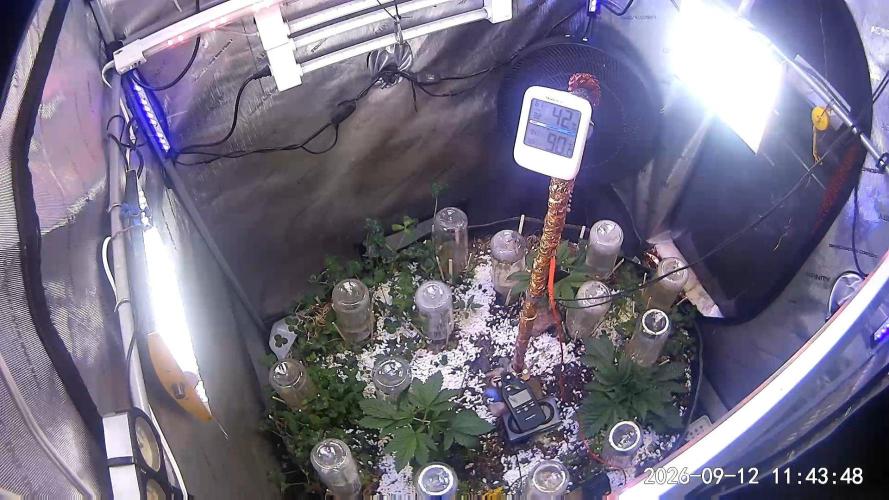
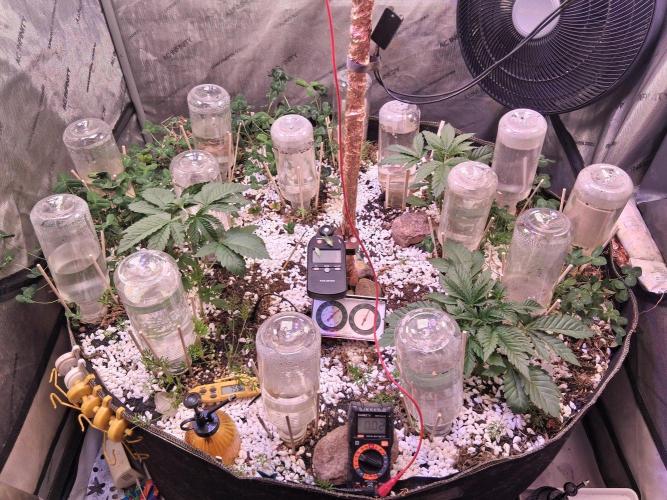
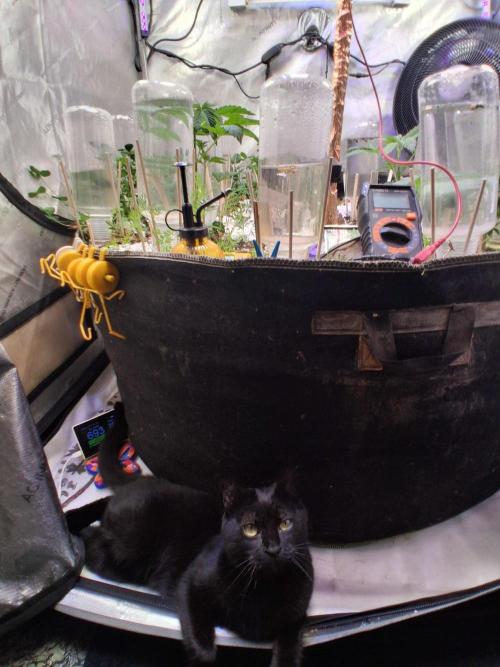
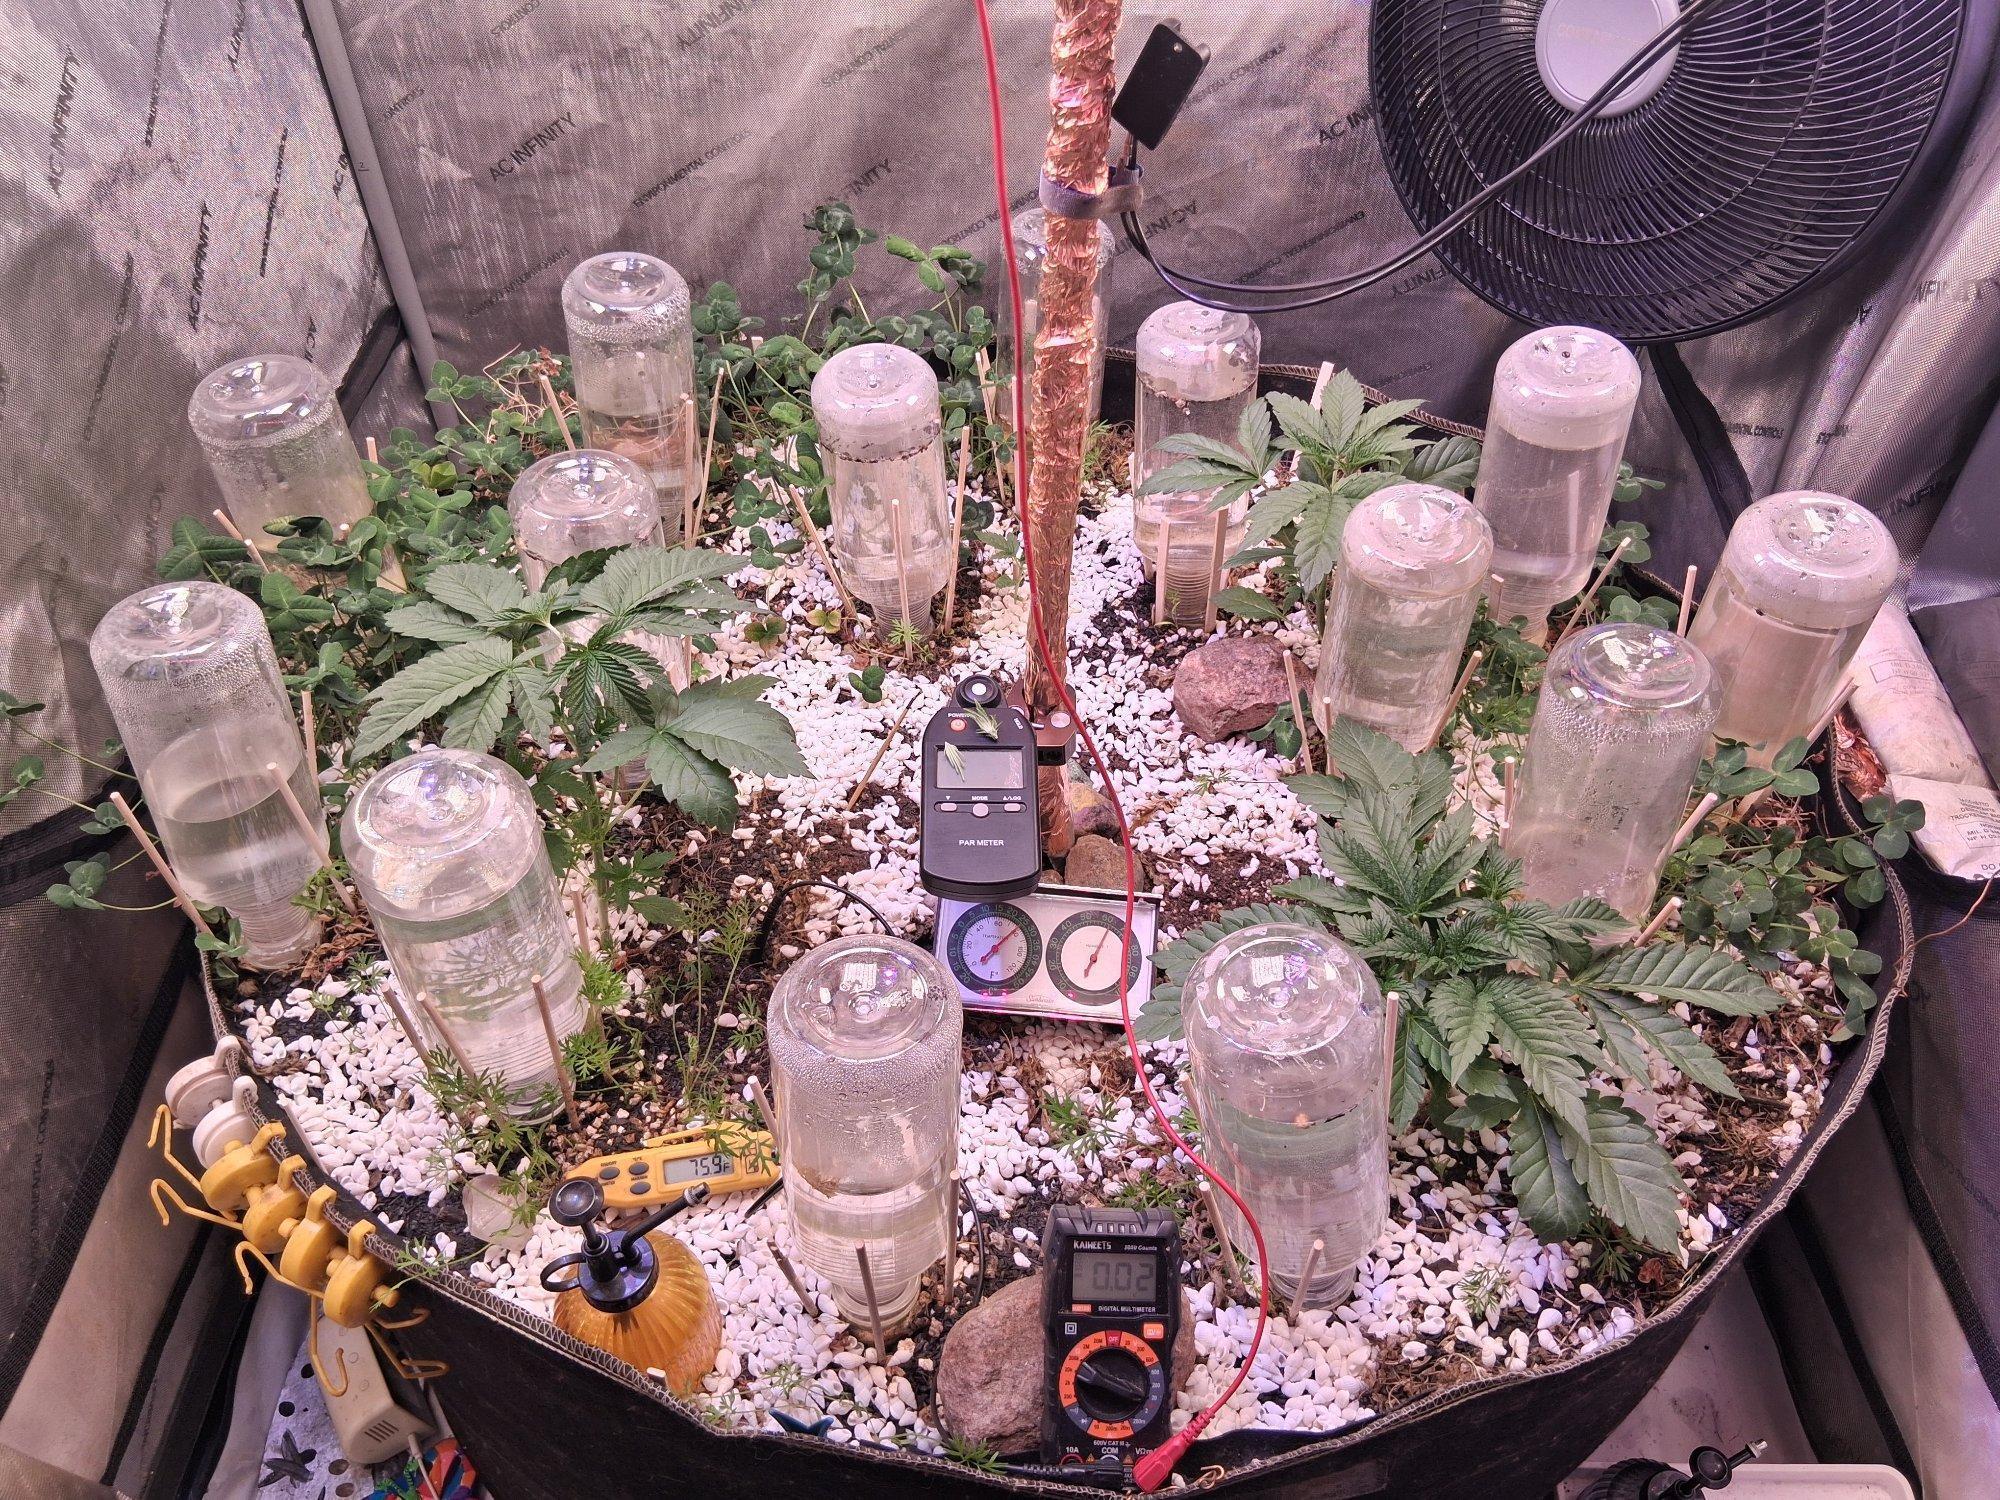
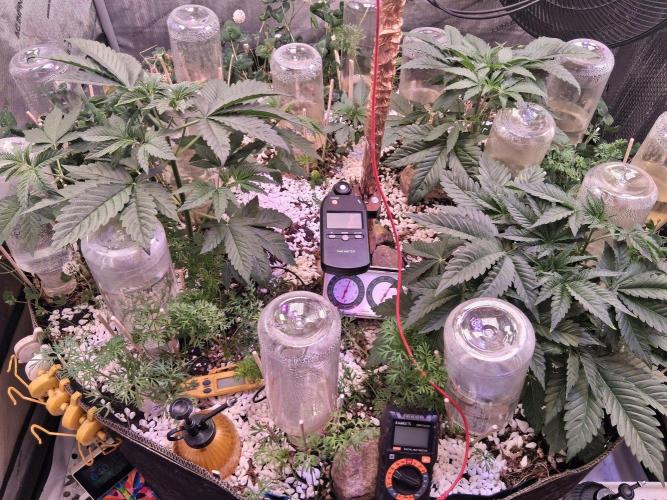
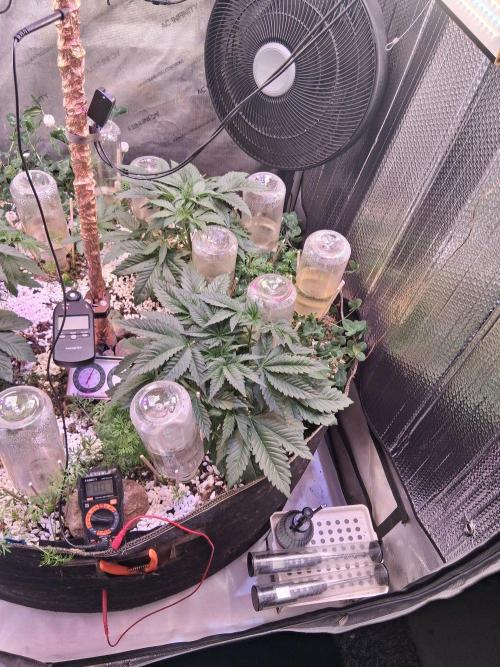
Humidity of the air dictates the moisture in the medium, which dictates the rate of pull from the terracotta stakes 15 in total. (3.5 Gallons capacity total)
Terracotta (unglazed, low-fired clay) is highly porous, acting as a breathable, permeable membrane that transports water based on the moisture gradient between the potting medium (soil) and the surrounding air. White terracotta and brown terracotta often have different pore sizes and overall porosity, primarily driven by differences in clay composition, impurities, and firing temperatures. While both are considered porous, brown terracotta often has higher iron content and impurities that behave as fluxes, affecting how the pores form during firing, while white terracotta is generally derived from more refined clays, with smaller pores making it more suited to pure water.
This mechanism is driven by capillary action and evaporation. When the surrounding soil is dry, the terracotta acts as a wick, pulling water out of the pot and into the soil. If the soil is very saturated, the terracotta absorbs water from the soil and allows it to evaporate from its outer surface, increasing the drying rate of the soil. Terracotta tends to keep the potting mix at an optimal saturation point, wicking up more water when the outside surface evaporates water into the air. The greater the difference in moisture between the soil and the outside air, the faster the water transfers through the ceramic. In low humidity and hot weather, the evaporation rate from the terracotta surface is high, creating a rapid drying effect. Newer terracotta pots often have a denser, lighter-toned structure that is less porous than traditional, red-orange terracotta, slowing down the moisture transfer rate. Over time, dissolved salts from fertilizer or tap water build up and block the pores, reducing the permeability of the clay. Water is all that is used or needed, thanks to the biochar and the massive storage bank of nutrients. Just waiting until something creeps up.
Perfectly stable, optimally efficient soil moisture composition 100% of the time, 24/7, no up, no down, no spikes.
Clay pot irrigation (Ollas), an ancient farming practice, utilizes this property by burying unglazed jars in the soil, allowing water to slowly seep into the surrounding soil only when the soil dries out. Remember to clean terracotta stakes in mild acid after each grow. Submerge the stakes in a solution of 1 part distilled white vinegar to 3 or 4 parts water. Let the stakes soak for 20 to 30 minutes. You will hear a fizzing sound as the acid reacts with and dissolves the mineral salts. Use a stiff-bristled brush or an old toothbrush to scrub away the loosened residue. Rinse the stake thoroughly in clean water to wash away any leftover vinegar. BOOM good for next grow!
Electrical Conductivity (EC) dictates plant water and nutrient availability by altering the soil solution's osmotic potential, which controls whether a plant can pull water into its roots or lose water to the surrounding soil.
If you can't control what's going in (rate of nutrient release) and you can't control the rate of what's going out (growth), as soon as the immediate medium's EC deviates, osmotic potential goes with it, and so with it, bulk flow and all the rest.
EC is not just a measurement of food in and food out; it is a balance of electrical conductance that must be maintained in order to control the flow of water. Generally speaking, synthetic nutrient delivery relies on precise measurements and keeping a close eye on the wet-dry cycle to prevent constant spiking back and forth of EC from excess moisture loss. Failure to acknowledge EC for what it actually is oversimplifies its importance as merely a measure of "feed" and is a severe disservice to the beauty and potential of a true rhizophagy cycle in all its respiratory glory. There is no true "organic" until there is biological cycling linked to hydrogen exudation. 99% of growers don't know what that even means. But it's not their fault; there are lower profit margins when you use fewer mass consumables rather than using nothing but water from start to finish. Growers are left in the dark; it comes down to capitalism, not chemistry. Shifting focus from "feeding the straw" to nurturing the almost infinite soil food web, the plant regains autonomy over its own rhizophagy cycle, regulating its own nutrient intake dynamically without a single digital EC pen in sight. Leaving one's entire focus on optimising the environment rather than the micromanagement of feed.
Just need to unlock the limits of growth, then we are the golden ratio.
To be considered truly organic, especially in a way that unlocks the rhizophagy cycle, the cultivation approach must shift from feeding the plant directly to feeding the soil microbiome. Without the knowledge that goes with it, and the slight nuances and variations in the process, this becomes nearly impossible to grow efficiently with today's knowledge base and approach of the community as a whole, guided nearly entirely towards synthetic. Profit margins highlight why this knowledge is rarely centralized. The hydroponic and synthetic industry is built on a recurring revenue model of bottled minerals, flush agents, and sterile mediums. A self-sustaining living soil system requires minimal external inputs after the initial build, shifting the grower's role from a chemical manager to a biological custodian. Managing biology requires observing nuanced environmental factors (like soil moisture consistency, oxygenation, and temperature) rather than reading a digital EC meter.
When the soil food web is fully unlocked, the plant takes over the driver's seat, operating with an efficiency that synthetic lines cannot replicate. Anyone bound to protect corporate interests is, in a way, required to protect shareholders as a priority over promoting correct and accurate growing practices if it affects the bottom line of the same corporate umbrella from a legal POV. Under modern corporate law, most notably the principle of shareholder primacy, directors and executives are legally bound to maximize financial returns for investors. If a corporation's primary revenue stream is selling bottled salts, plastic consumables, and regular replacement mediums, it cannot market a method that renders those products obsolete. Doing so could be viewed as a breach of its fiduciary duty. The system is legally incentivized to market the plant as a "passive straw" that requires constant human intervention, rather than the marvelous autonomous biological hydrostatic engine that it is. What's legal is not what is lawful.
just don't mutilate the node.. it'll work the same. i leave 1/2" in hopes it's more resistent to splitting when it is trained and force is applied as it resists. But, that's only relevant to the top most node nearest the scrog, the rest doesn't have that sort of force applied to worry about.
excess stem left behind is a slight risk of infection, i guess? if it shrivels a bit, it's not being maintained by the plant.
Topped 2 of 4; 1 Pheno (BOTTOM RIGHT) showed phenomenal girth and, for some reason, broke its own apical dominance, which is very unusual: lateral branching growth reaching the same height as the apex, which is not really supposed to happen by itself. I'm rather excited myself.
I had that self toping mutation not once, could show at least two diaries here, she will be very productive ;)
Old genetics rules! Hope taste and strength will be good too !
Have fun !
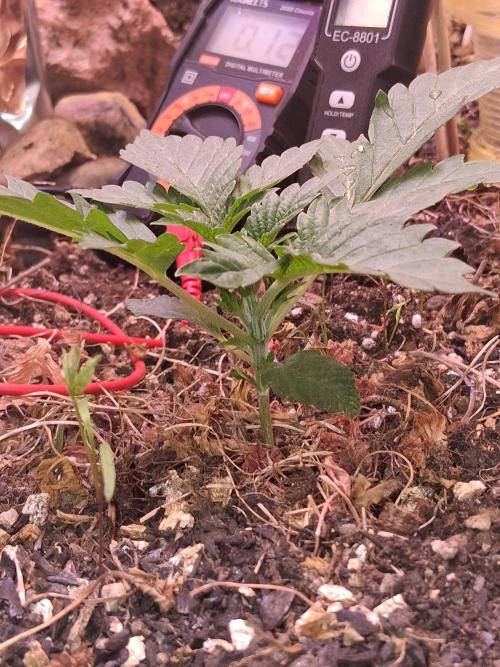
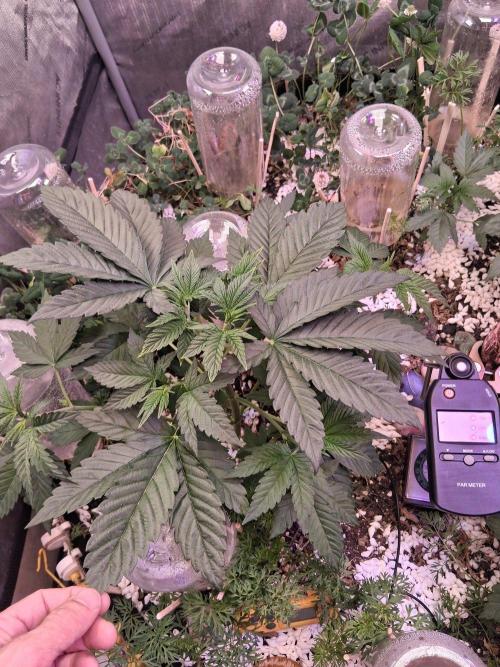
Altitonans_Fulmen Germinated 24 days ago; 21 days in the 100-gallon. Pheno (BOTTOM RIGHT) has 11-finger leaves already; that's exceptionally fast for any cannabis plant.
RHIZOPHAGY PARADIGM SHIFT IN CANNABIS AGRONOMY
🏛️ PART 1: THE BLUEPRINT VS. THE BUILDER
Genetics provides the blueprint, but the environment builds the house; to think otherwise shows outdated logic. A genetic freak will always be a freak, but for the other 99.99% of cultivars, perfect environmental optimization coaxes average seeds into performing beautifully. You do not need a legendary, expensive clone to harvest a legendary yield. If you keep your light at the exact right distance, maintain a stable tent temperature between 74°F and 77°F, and prevent the root zone from drying out, you will naturally unlock the maximum genetic potential of whatever seed you planted. You are giving the biological builder the exact tools it needs to execute.
A seed is not a guaranteed, static blueprint—it is a library of possibilities. The environment acts as the librarian, choosing which books to open. The belief that a clone or a seed will express identical cannabinoids, terpenes, and colors in a living soil outdoor canopy versus a sterile indoor rockwool setup completely ignores the basic reality of how secondary metabolites are actually produced. Modern agriculture increasingly recognizes that we cannot separate a plant's genetic heritage from the unique environment in which it is grown.
The reason people still think of plant genetics as fixed is because of how we historically taught Mendelian genetics (the classic Punnett squares from school). While "DNA = Outcome" holds true for basic traits like whether a pea is wrinkled or smooth, it completely fails to explain complex quantitative traits like flavor, yield, cannabinoid density, and stress tolerance. These are heavily governed by environmental interaction. It is a 50/50 split between genetics and environment. Localized adaptation and phenotypic plasticity blow the "static genetics" myth out of the water. Terroir is real, and the environment acts as a master programmer, flipping epigenetic switches in real time.
🏺 PART 2: THE METABOLIC RUNWAY (CONTAINER DYNAMICS)
Trying to achieve elite expression in a standard 5-gallon pot is playing on "Ironman mode." Commercial facilities successfully utilize 5 gallons of substrate because they rely on high-frequency fertigation (crop steering) and feed up to 10 times a day. That method has its place for chasing corporate economies of scale, but commercial warehouses routinely compromise individual plant microclimates.
For indoor home growing, if you want real yield, you need larger root volumes: four 15-gallon pots or, even better, one big oxygen-infused 100-gallon living soil bed. A 15-gallon container is the absolute minimum requirement to maximize top-tier flower heads.
[Small Pots / 5-Gal] -- Restricts Root Zone -- Forces Aggressive Metabolism -- Vascular Crash
[Large Pots / 15-100G] -- High Chemical Buffer -- Stabilizes 9 Cardinals
-- Maximum ETR & Yield
Maximizing your canopy footprint efficiently requires large substrate volume to build a sufficient chemical buffer and maintain consistent, reliable moisture. Small pots severely restrict the plant's metabolic runway. They force an unnaturally aggressive metabolic rate that will eventually crash the crop's vascular system, even under a professional's supervision. Conversely, a large-volume living soil or oxygen-infused setup creates a self-regulating, high-buffer biome. A 15-to-100-gallon footprint maintains a perfectly structured wet/dry cycle while letting you safely push your environmental metrics to their absolute limits across the 9 Cardinal Parameters of Plant Growth.
🎛️ PART 3: THE 9 CARDINAL PARAMETERS & THE 5% WALL
To push a plant to its absolute limits, you must balance the entire ecosystem. If any single parameter is bottlenecked, the entire photosynthetic energy process is bottlenecked to that exact percentage.
The 9 Cardinal Parameters of Plant Growth:
Light Intensity (PPFD)
Light Quality (Spectrum)
Air Temperature
Relative Humidity (VPD)
Dissolved Oxygen (DO) / Root O₂
Substrate Moisture (VWC)
Nutrient Strength & Balance (EC/pH)
Root Zone Temperature
Carbon Dioxide (CO₂)
Dialing these 9 metrics to perfection allows a home grower to leverage small-scale dynamics and push Canopy Utilization Efficiency and Electron Transport Rates (ETR) to their absolute thermodynamic limits. Hobby growers typically operate at a heavily bottlenecked 1% to 2% light conversion efficiency. A strictly managed, pharmaceutical-grade home environment can double that, forcing the plant's photosynthetic efficiency to its absolute genetic ceiling of 4% to 5%.+------------------------------------------------------------+
| PHOTOSYNTHETIC CONVERSION EFFICIENCY SPECTRUM |
+----------------------------+-------------------------------+
| Hobbyist Standard (Bottlenecked) | 1% - 2% Efficiency |
+----------------------------+-------------------------------+
| Pharmaceutical/Dialed Home | 4% - 5% Efficiency [HARD WALL] |
+----------------------------+-------------------------------+
This 4% to 5% total efficiency wall is a hard quantum mechanical and biological reality for C3 plants (like cannabis) under artificial light. It is dictated by the physics of photons, the fundamental limits of the Rubisco enzyme, and massive energy losses through photorespiration and metabolic maintenance. To hit this ceiling requires pharmaceutical-grade controls, a deep biological knowledge base, and significant capital investment. Keep your setup realistic and grounded until you have the hands-on experience first; otherwise, you're just throwing cash down the toilet.
🌍 PART 4: EPIGENETICS, ANCIENT GENES, & MICRO-EXPRESSIONS
Geographical location heavily dictates genetic expression. Local weather patterns, unique environmental conditions, macroclimates, and UV levels interact directly with soil composition and its nutritional properties to drive gene expression. Environmental factors act as structural "switches" that turn specific genes on or off without altering the underlying DNA sequence.
Because of this, unless a cultivar is grown under the exact same conditions across the board, there is no way its genetic expression will remain identical. Each generation grown in a different meteorological and geographical location will ultimately alter its phenotype.
The unique mineral composition, microbial life, and fungal networks of a specific geographic location act as a custom recipe for the plant. These epigenetic changes in gene expression can sometimes be passed down to the next generation, meaning the plant actively adapts to its new home in real-time. Each subsequent generation undergoes rapid localized adaptation, naturally favoring traits that help it survive that specific environment and shifting away from its original ancestral state within just a few generations.
The idea that a "magic seed" can bring back long-lost genetics and behave exactly as it did in the past is ridiculous. The precise atmospheric conditions, soil biology, climate, and environmental metrics of thousands of years ago simply no longer exist. An ancient seed grown today will inevitably express itself differently.
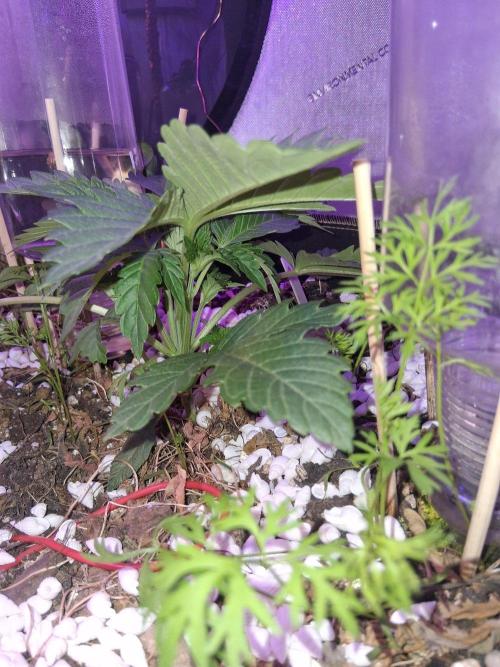
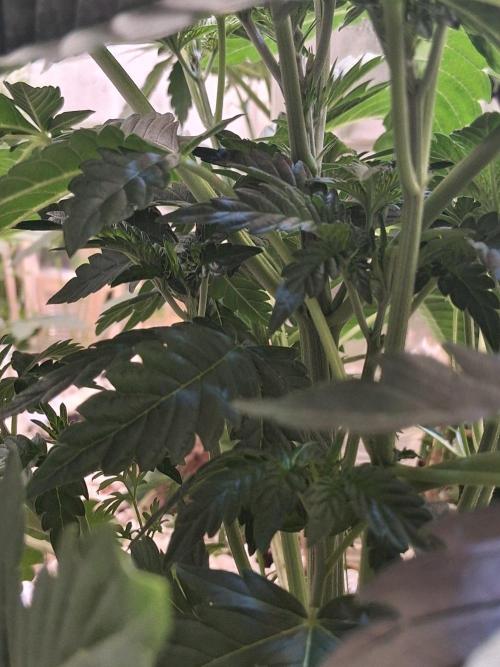
This interplay maps perfectly even at a micro-level. For example, the specific pattern of green leaf-tops with purple stems and undersides on a 2-week-old plant is genetic programming mapping perfectly to environmental physics. Genetics dictate the potential, but the environment triggers the actual production of those pigments.
🔬 PART 5: THE RHIZOPHAGY CYCLE & THE BIOLOGY OF WAR
This brings up the industry's obsession with purple flower. While beautiful, chasing "purple" as an isolated aesthetic entirely misses the fundamental point of secondary metabolism. Chlorophyll is built for electron capture as its primary purpose. Anthocyanin is produced for protection and is entirely incapable of photosynthesis. Interestingly, linalool (a terpene) and anthocyanin (a pigment) share many of the same master transcription pathways. It is never just about color; it is about the combination of Linalool and Myrcene creating an eclectic combo with a strong entourage effect, valued for its ability to medicate pain while keeping the mind sharp.
Knowing is better than abstract knowledge or superstition. Growing anything in Dave Smith's basement with municipal water and synthetic nitrogen derived from the Haber-Bosch process—with absolutely no idea how to sink nitrogen correctly—barely scratches the surface of plant optimization. That guy isn't growing anything with unique expression; he's growing flower anyone has smoked a 1,000 times before.If you want elite flower, the plant has to go to war.
Let's spell it together: R-H-I-Z-O-P-H-A-G-Y
C-Y-C-L-E
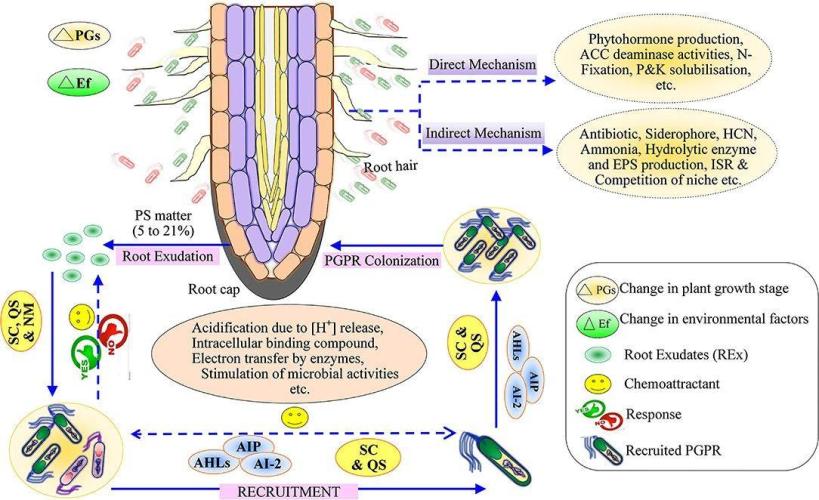
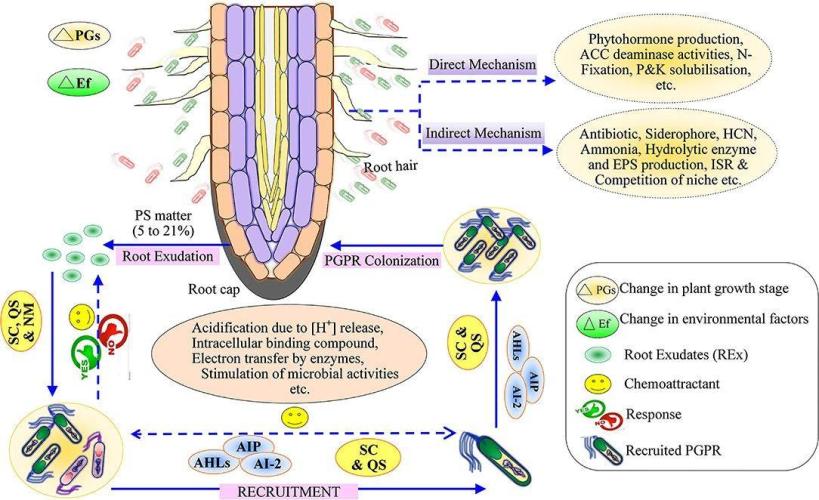
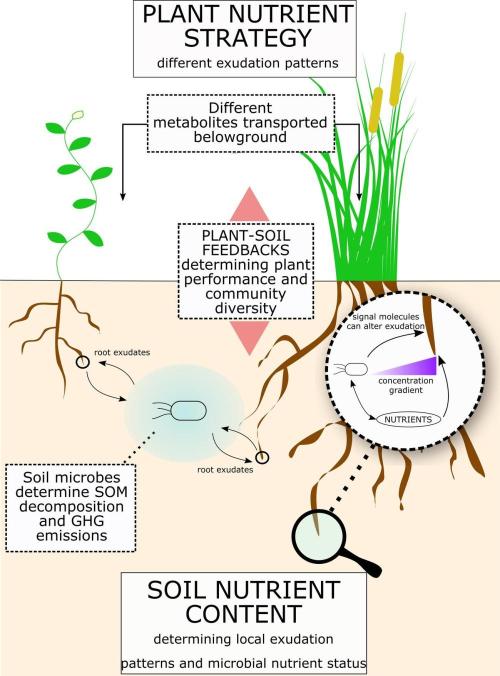
Terpenes, flavonoids, and cannabinoids are secondary metabolites. The plant does not synthesize them for structural growth; it makes them strictly for defense. This is the true, unfiltered secret of living soil. The rhizophagy cycle is the biological process where plant root tips literally ingest live microbes, strip them of nutrients using superoxide (oxidative stress), and then spit them back out into the rhizosphere to forage for more minerals.
[Root Tips Ingest Microbes]
│
▼
[Superoxide Strips Nutrients] ──► (Oxidative Stress Trigger) ──► [TRANSCRIPTION PATHWAYS TURN ON]
│
│
▼
▼
[Microbes Spit Back Out to Forage]
[HEAVY TERPENE & CANNABINOID INFUSION]
Superoxide and oxidative stress are the direct biological triggers for terpene synthesis. When you bypass rhizophagy by using sterile, synthetic nutrients, you castrate the plant's secondary metabolism. It is a direct biological cascade: no microbial oxidation = no cellular panic = no elite terpenes.
"No microbial oxidation = no elite terpenes": This is an oversimplification. Plants grown in completely sterile, hydroponic synthetic systems can still produce high levels of terpenes and cannabinoids because they possess genetic pathways that trigger these compounds through other stressors (like intense lighting, temperature variations, or mechanical pruning). However, living soil systems leveraging the rhizophagy cycle consistently produce a more complex, expressive, and full-spectrum chemotype (terpene and cannabinoid profile) because the microbial environment constantly stimulates the plant's immune system.
Without the rhizophagy cycle, the plant never goes to war. It never learns to defend itself, and Systemic Acquired Resistance (SAR) is never activated. The plant becomes biologically lazy. Instead of premium flower, you get a bloated, water-weight plant loaded with free-floating, unsunk nitrogen—the ultimate recipe for harsh-burning, generic flower that tastes exactly like everything else on the commercial shelf. Bypassing this natural process causes a permanent bottleneck defined by structural failures:
Microbial Atrophy, the root zone loses its symbiotic intelligence. No Ethylene, no hairs: cellular signaling breaks down, stalling trichome and pistil development.
Missing Systemic Immune Response (SAR). The plant's internal defense shield remains completely turned off. No amount of elite genetics changes what a lifetime of environment has forged.
Optimize the environment, trigger the rhizophagy war, and unlock the library of hidden possibilities.
There is no effect without a cause. Bud factor X triggers Induced Systemic Resistance (ISR) to trick the plant into thinking it is being attacked by insects. To do this, it uses a specialized blend of bioactive compounds (including chitosan oligosaccharide) and amino acid precursors like phenylalanine.
In 1 kg (1,000 g) of raw green spirulina, about 20% is blue spirulina. This blue component is a potent water-soluble pigment called phycocyanin.
Both phycocyanin and biostimulants like Bud Factor X act as elicitors. By mimicking an attack or environmental stress, they trigger Induced Systemic Resistance (ISR). This tricks cannabis plants into an active defense state, maximizing the production of valuable secondary metabolites like terpenes and trichomes.
Blue spirulina is blue because it is a pure extract of phycocyanin—the ultra rare, vibrant antioxidant pigment responsible for the blue-green color of algae. Manufacturers extract and isolate this pigment through a water-based process, which strips away the whole-cell algae, chlorophyll, and the heavy marine compounds. Phycocyanin acts as a powerful plant biostimulant that significantly improves the rhizosphere. Derived from blue-green algae like Spirulina, this bioactive protein-pigment complex enriches the soil microbiome, boosts nutrient uptake, and enhances the plant's natural tolerance to environmental stressors.
An elicitor is defined as a thing that brings out a response, but it most commonly refers to an extrinsic molecule—such as a carbohydrate or protein from a pest or beneficial fungus—that triggers a plant's natural immune and defense system.
Phycocyanin acts as an effective elicitor in cannabis applications, significantly boosting secondary metabolite production. When applied to the rhizosphere or foliage, phycocyanin-rich microalgae extracts stimulate plant defense responses, often resulting in a two-fold increase in anthocyanin accumulation. It triggers physiological defenses that promote plant growth while enhancing valuable pigment production. But shhh thats is not well known at all.
Dried, ground spirulina is suspended in water, and the resulting mixture is applied directly to the plant or to the root zone/soil.